16 Forensic Anthropology
Ashley Kendell; Alex Perrone; and Colleen Milligan
Student contributors to this chapter: Amelia Roberts, Elyse Racicot, Emmanuelle Hunter
Learn more about authors and editors, Hess’ student contributions, and versioning history.
Content Warning and Disclaimer: This chapter includes images of human remains as well as discussions centred on human skeletal analyses. All images are derived from casts, sketches, nonhuman skeletal material, as well as non-Indigenous skeletal materials curated within the CSU, Chico Human Identification Lab, and the Hartnett-Fulginiti donated skeletal collection.
Learning Objectives
- Define forensic anthropology as a subfield of biological anthropology.
- Describe the seven steps carried out during skeletal analysis.
- Outline the four major components of the biological profile.
- Contrast the four categories of trauma.
- Explain how to identify the different taphonomic agents that alter bone.
- Discuss ethical considerations for forensic anthropology.
Forensic anthropology is a subfield of biological anthropology and an applied area of anthropology. Forensic anthropologists use skeletal analysis to gain information about humans in the present or recent past, then they apply this information within a medicolegal context. This means that forensic anthropologists specifically conduct their analysis on recently deceased individuals (typically within the last 50 years) as part of investigations by law enforcement. Forensic anthropologists can assist law enforcement agencies in several different ways, including aiding in the identification of human remains whether they are complete, fragmentary, burned, scattered, or decomposed. Additionally, forensic anthropologists can help determine what happened to the deceased at or around the time of death as well as what processes acted on the body after death (e.g., whether the remains were scattered by animals, whether they were buried in the ground, or whether they remained on the surface as the soft tissue decomposed).
Many times, because of their expertise in identifying human skeletal remains, forensic anthropologists are called to help with outdoor search-and-recovery efforts, such as locating remains scattered across the surface or carefully excavating and documenting buried remains. In other cases, forensic anthropologists recover remains after natural disasters or accidents, such as fire scenes, and can help identify whether each bone belongs to a human or an animal. Forensic anthropology spans a wide scope of contexts involving the law, including incidences of mass disasters, genocide, and war crimes.
A point that can be somewhat confusing for students is that although the term forensic is included in this subfield of biological anthropology, there are many forensic techniques that are not included in the subfield. Almost exclusively, forensic anthropology deals with skeletal analysis. While this can include the comparison of antemortem (before death) and postmortem (after death) radiographs to identify whether remains belong to a specific person, or using photographic superimposition of the cranium, it does not include analyses beyond the skeleton. For example, blood-spatter analysis, DNA analysis, fingerprints, and material evidence collection do not fall under the scope of forensic anthropology.
So, what can forensic anthropologists glean from bones alone? Forensic anthropologists can address a number of questions about a human individual based on their skeletal remains. Some of those questions are as follows: How old was the person? Was the person biologically male or female? How tall was the person? What happened to the person at or around their time of death? Were they sick? The information from the skeletal analysis can then be matched with missing persons records, medical records, or dental records, aiding law enforcement agencies with identifications and investigations.
Skeletal Analysis
Forensic anthropology relies on skeletal analysis to reveal information about the deceased. The methodology and approaches outlined below are specific to the United States. Forensic anthropological methods differ depending on the country conducting an investigation. In the United States, there are typically seven steps or questions to the process:
- Is it bone?
- Is it human?
- Is it modern or archeological?
- How many individuals are present or what is the minimum number of individuals (MNI)?
- Who is it?
- Is there evidence of trauma before or around the time of death?
- What happened to the remains after death?
Is It Bone?
One of the most important steps in any skeletal analysis starts with determining whether or not material suspected to be bone is in fact bone. Though it goes without saying that a forensic anthropologist would only carry out analysis on bone, this step is not always straightforward. Whole bones are relatively easy to identify, but determining whether or not something is bone becomes more challenging once it becomes fragmentary. As an example, in high heat such as that seen on fire scenes, bone can break into pieces. During a house fire with fatalities, firefighters watered down the burning home. After the fire was extinguished, the sheetrock (used to construct the walls of the home) was drenched and crumbled. The crumbled sheetrock was similar in colour and form to burned, fragmented bone, therefore mistakable for human remains (Figure 16.1). Forensic anthropologists on scene were able to separate the bones from the construction material, helping to confirm the presence of bone and hence the presence of individual victims of the fire. In this case, forensic anthropologists were able to recognize the anatomical and layered structure of bone and were able to distinguish it from the uniform and unlayered structure of sheetrock.
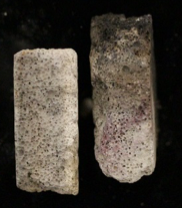
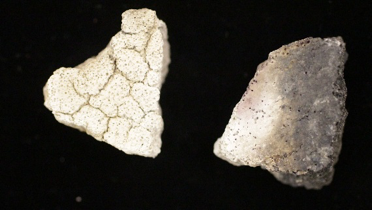
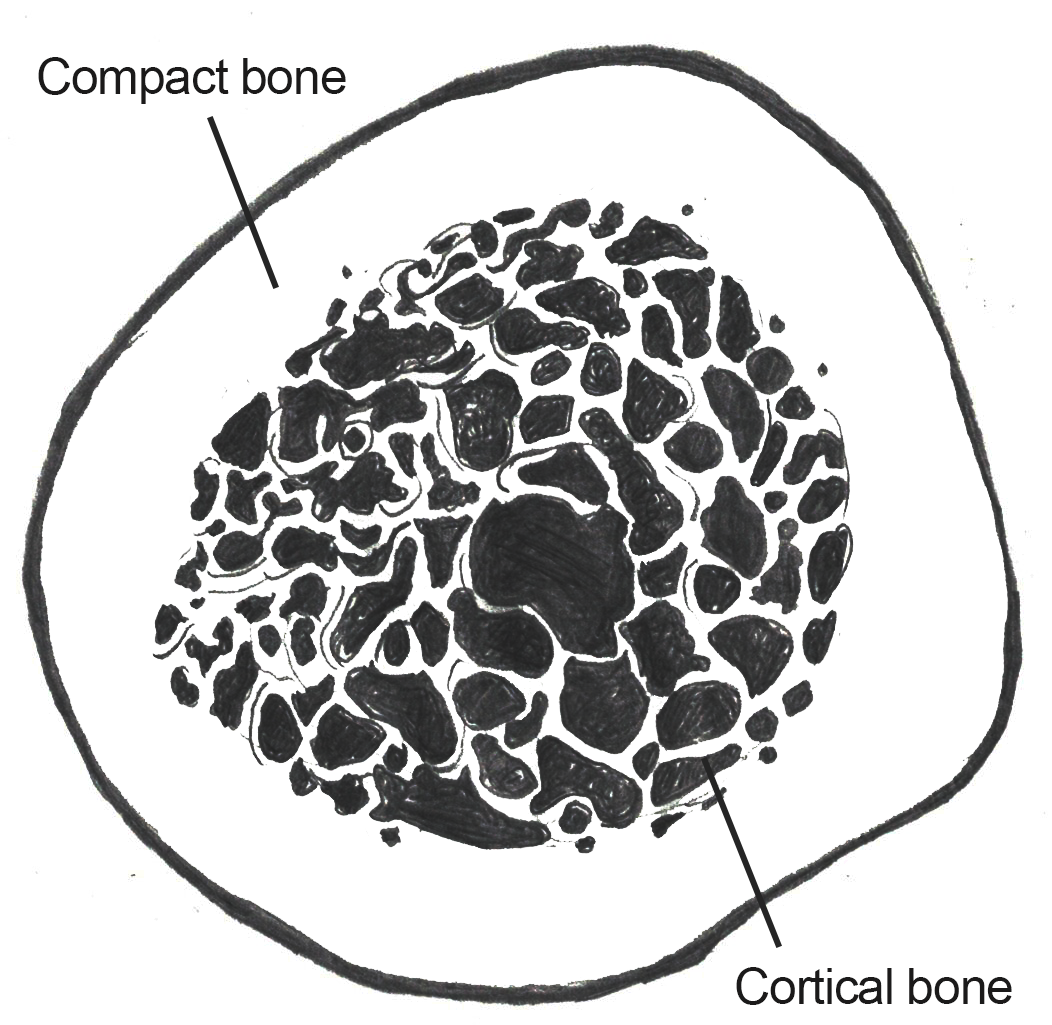
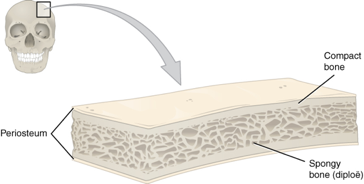
As demonstrated by the example above, both the macrostructure (visible with the naked eye) and microstructure (visible with a microscope) of bone are helpful in bone identification. Bones are organs in the body made up of connective tissue. The connective tissue is hardened by a mineral deposition, which is why bone is rigid in comparison to other connective tissues such as cartilage (Tersigni-Tarrant and Langley 2017, 82–83; White and Folkens 2005, 31). In a living body, the mineralized tissue does not make up the only component of bone—there are also blood, bone marrow, cartilage, and other types of tissues. However, in dry bone, two distinct layers of the bone are the most helpful for identification. The outer layer is made up of densely arranged osseous (bone) tissue called compact (cortical) bone. The inner layer is composed of much more loosely organized, porous bone tissue whose appearance resembles that of a sponge, hence the name spongy (trabecular) bone. Knowing that most bone contains both layers helps with the macroscopic identification of bone (Figures 16.2, 16.3). For example, a piece of coconut shell might look a lot like a fragment of a human skull bone. However, closer inspection will demonstrate that coconut shell only has one very dense layer, while bone has both the compact and spongy layers.
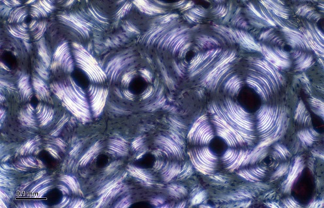
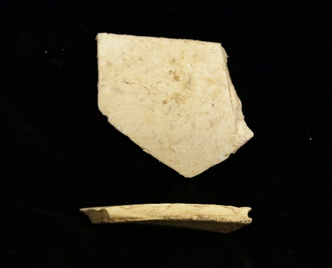
The microscopic identification of bone relies on knowledge of osteons, or bone cells (Figure 16.4). Under magnification, bone cells are visible in the outer, compact layer of bone. The bone cells are arranged in a concentric pattern around blood vessels for blood supply. The specific shape of the cells can help differentiate, for example, a small piece of PVC (white plastic) pipe from a human bone fragment (Figure 16.5).
Is It Human?
Once it has been determined that an object is bone, the next logical step is to identify whether the bone belongs to a human or an animal. Forensic anthropologists are faced with this question in everyday practice because human versus nonhuman bone identification is one of the most frequent requests they receive from law enforcement agencies.
There are many different ways to distinguish human versus nonhuman bone. The morphology (the shape/form) of human bone is a good place for students to start. Identifying the 206 bones in the adult human skeleton and each bone’s distinguishing features (muscle attachment sites, openings and grooves for nerves and blood vessels, etc.) is fundamental to skeletal analysis.
Nevertheless, there are many animal bones and human bones that look similar. For example, the declawed skeleton of a bear paw looks a lot like a human hand, pig molars appear similar to human molars, and some smaller animal bones might be mistaken for those of an infant. To add to the confusion, fragmentary bone may be even more difficult to identify as human or nonhuman. However, several major differences between human and nonhuman vertebrate bone help distinguish the two.
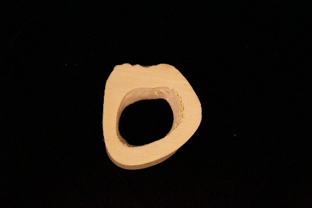
Forensic anthropologists pay special attention to the density of the outer, compact layer of bone in both the cranium and in the long bones. Human cranial bone has three distinctive layers. The spongy bone is sandwiched between the outer (ectocranial) and inner (endocranial) compact layers. In most other mammals, the distinction between the spongy and compact layers is not always so definite. Secondly, the compact layer in nonhuman mammal long bones can be much thicker than observed in human bone. Due to the increased density of the compact layer, nonhuman bone tends to be heavier than human bone (Figure 16.6).
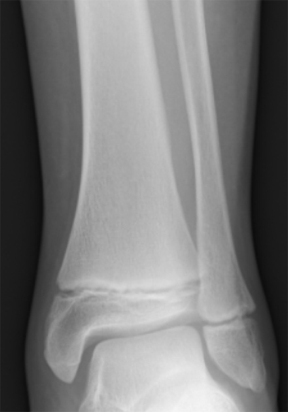
The size of a bone can also help determine whether it belongs to a human. Adult human bones are larger than subadult or infant bones. However, another major difference between human adult bones and those of a young individual or infant human can be attributed to development and growth of the epiphyses (ends of the bone). The epiphyses of human subadult bones are not fused to the shaft (Figure 16.7). Therefore, if a bone is small and it is suspected to belong to a human subadult or infant, the epiphyses would not be fused. Many small animal bones appear very similar in form compared to adult human bones, but they are much too small to belong to an adult human. Yet they can be eliminated as subadult or infant bones if the epiphyses are fused to the shaft.
Is It Modern or Archaeological?
Forensic anthropologists work with modern cases that fall within the scope of law enforcement investigations. Accordingly, it is important to determine whether discovered human remains are archaeological or forensic in nature. Human remains that are historic are considered archeaological. The scientific study of human remains from archaeological sites is called bioarchaeology.
Dig Deeper: Bioarchaeology
For readers who are interested in the sister subfield of bioarchaeology, which studies human remains and material culture from the past, please refer to chapter 8 of Bioarchaeology: Interpreting Human Behaviour from Skeletal Remains, in TRACES: An Open Invitation to Archaeology (Blatt, Michael, and Bright forthcoming).
A forensic anthropologist should begin their analysis by reviewing the context in which the remains were discovered. This will help them understand a great deal about the remains, including determining whether they are archaeological or forensic in nature as well as considering legal and ethical issues associated with the collection, analysis, and storage of human remains (see “Ethics and Human Rights” section of this chapter for more information).
The “context” refers to the relationship the remains have to the immediate area in which they were found. This includes the specific place where the remains were found, the soil or other organic matter immediately surrounding the remains, and any other objects or artifacts in close proximity to the body. For example, imagine that a set of remains has been located during a house renovation. The remains are discovered below the foundation. Do the remains belong to a murder victim? Or was the house built on top of an ancient burial ground? Observing information from the surroundings can help determine whether the remains are archaeological or modern. How long ago was the foundation of the house erected? Are there artifacts in close proximity to the body, such as clothing or stone tools? These are questions about the surroundings that will help determine the relative age of the remains.
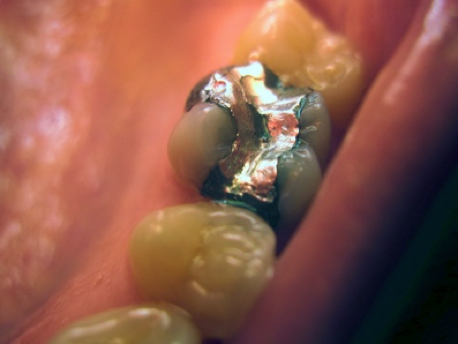
Clues directly from the skeleton may also indicate whether the remains are archaeological or modern. For example, tooth fillings can suggest that the individual was alive recently (Figure 16.8). In fact, filling material has changed over the decades, so the specific type of material used to fix a cavity can be matched with specific time periods. Gold was used in dental work in the past, but more recently composite (a mixture of plastic and fine glass) fillings have become more common.
How Many Individuals Are Present?
What Is MNI?
Another assessment that an anthropologist can perform is the calculation of the number of individuals in a mixed burial assemblage. Because not all burials consist of a single individual, it is important to burial assemblage be able to estimate the number of individuals in a forensic context. Quantification of the number of individuals in a burial assemblage can be done through the application of a number of methods, including the following: the Minimum Number of Individuals (MNI), the Most Likely Number of Individuals (MLNI), and the Lincoln Index (LI). The most commonly used method in biological anthropology, and the focus of this section, is determination of the MNI.
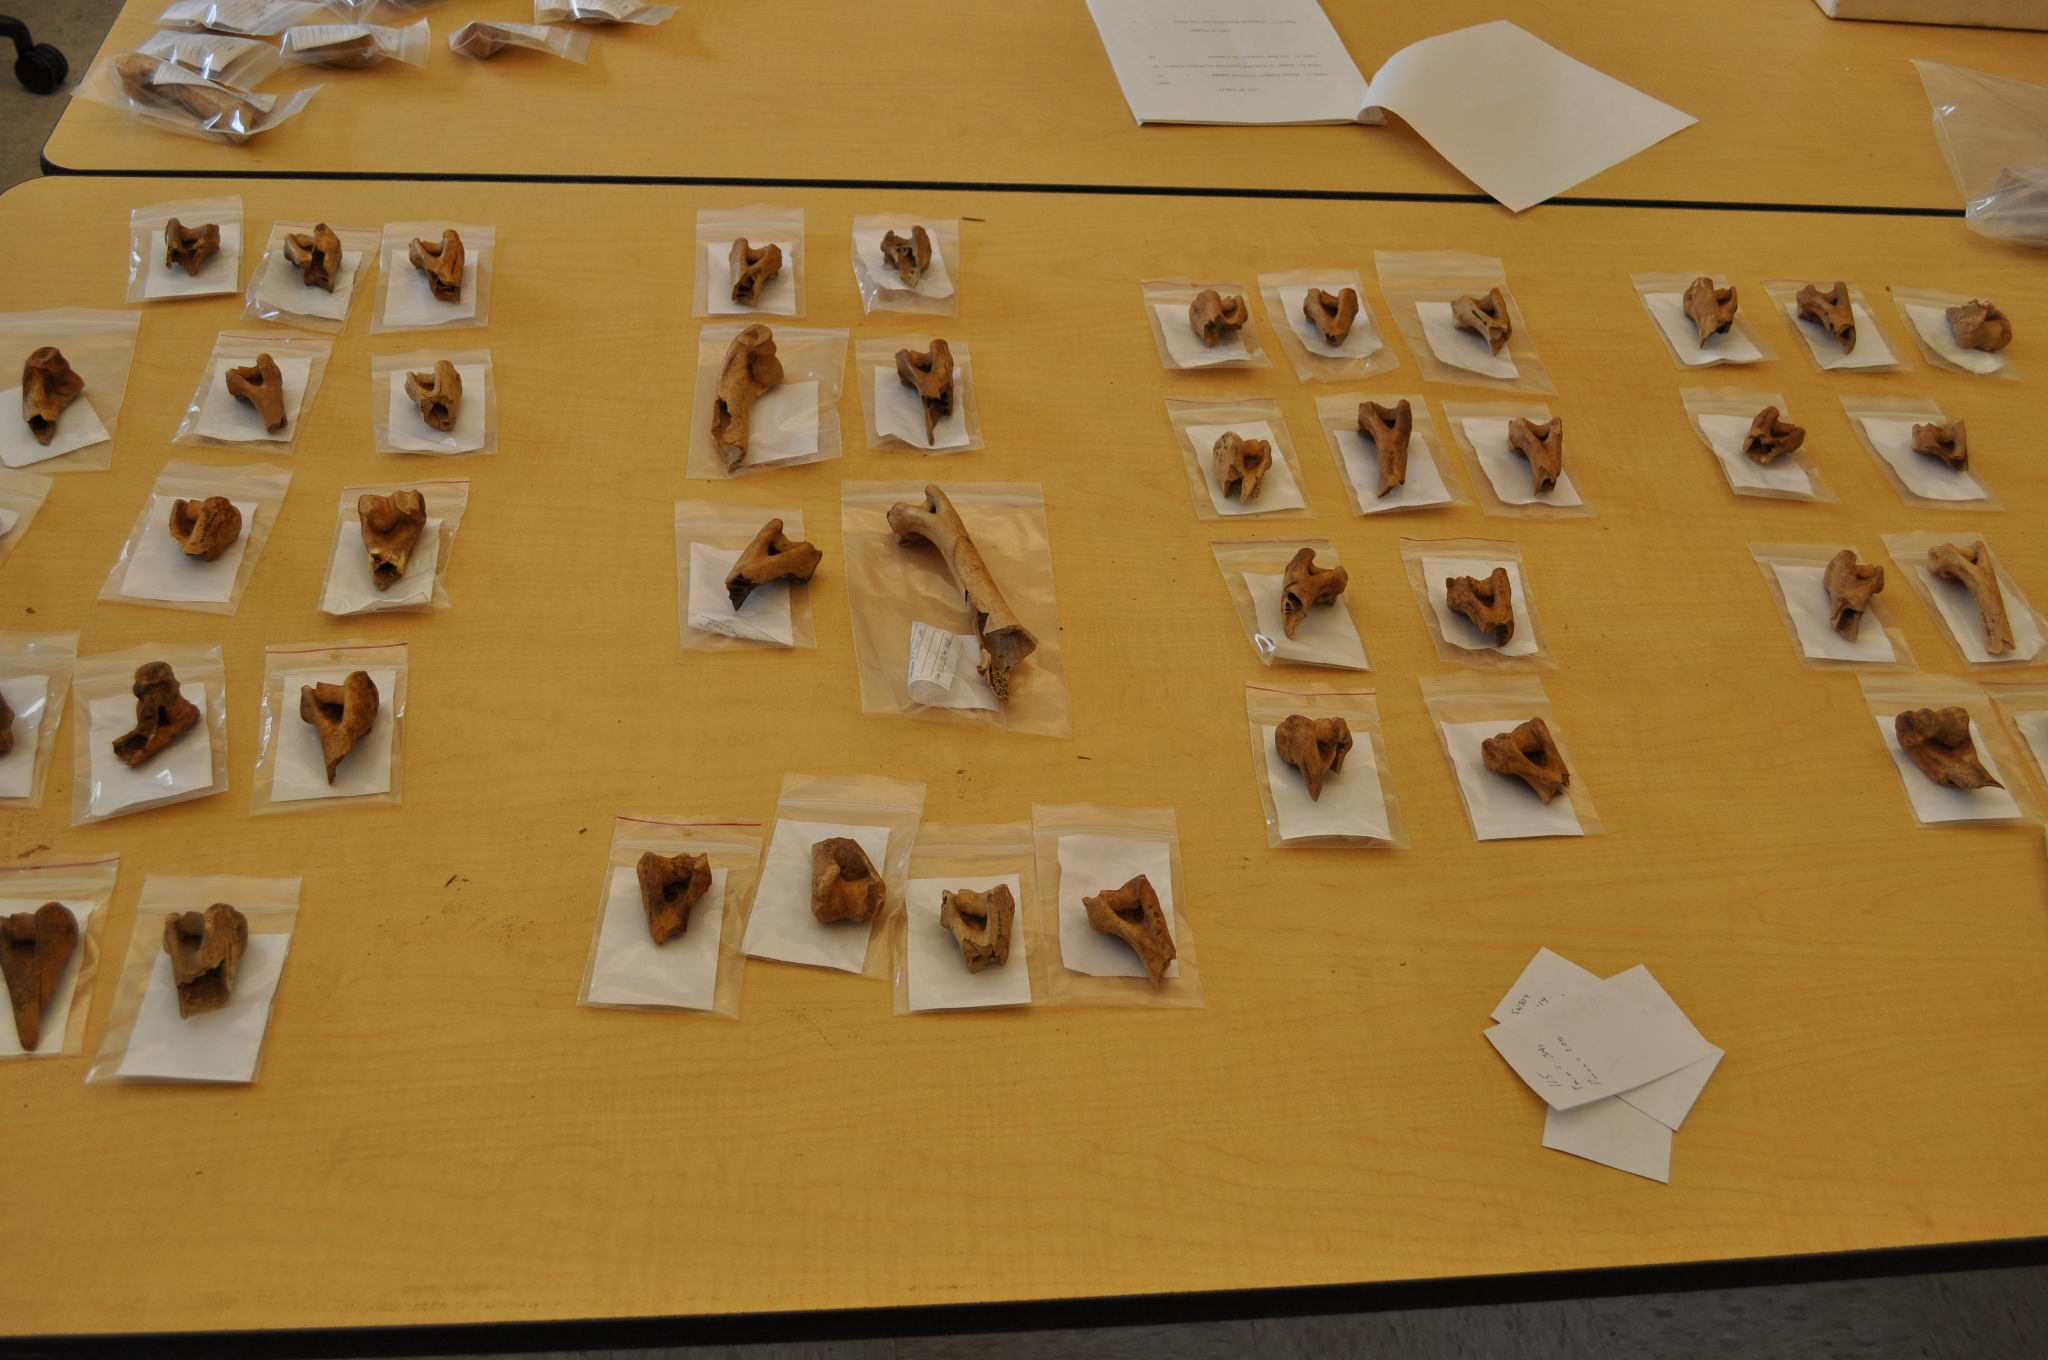
The MNI presents “the minimum estimate for the number of individuals that contributed to the sample” (Adams and Konigsberg 2008, 243). Many methods of calculating MNI were originally developed within the field of zooarchaeology for use on calculating the number of individuals in faunal or animal assemblages (Adams and Konigsberg 2008, 241). What MNI calculations provide is a lowest possible count for the total number of individuals contributing to a skeletal assemblage. Traditional methods of calculating MNI include separating a skeletal assemblage into categories according to the individual bone and the side the bone comes from and then taking the highest count per category and assigning that as the minimum number (Figure 16.9).
Why Calculate MNI?
In a forensic context, the determination of MNI is most applicable in cases of mass graves, commingled burials, and mass fatality incidents. The term commingled is applied to any burial assemblage in which individual skeletons are not separated into separate burials. As an example, the authors of this chapter have observed commingling of remains resulting from mass fatality wildfire events. Commingled remains may also be encountered in events such as a plane or vehicle crash. It is important to remember that in any forensic context, MNI should be referenced and an MNI of one should be substantiated by the fact that there was no repetition of elements associated with the case.
Constructing the Biological Profile
Who Is It?
“Who is it?” is one of the first questions that law enforcement officers ask when they are faced with a set of skeletal remains. To answer this question, forensic anthropologists construct a biological profile (White and Folkens 2005, 405). A biological profile is an individual’s identifying characteristics, or biological information, which include the following: biological sex, age at death, stature, population affinity, skeletal variation, and evidence of trauma and pathology.
Assessing Biological Sex
Assessment of biological sex is often one of the first things considered when establishing a biological profile because several other parts, such as age and stature estimations, rely on an assessment of biological sex to make the calculations more accurate.
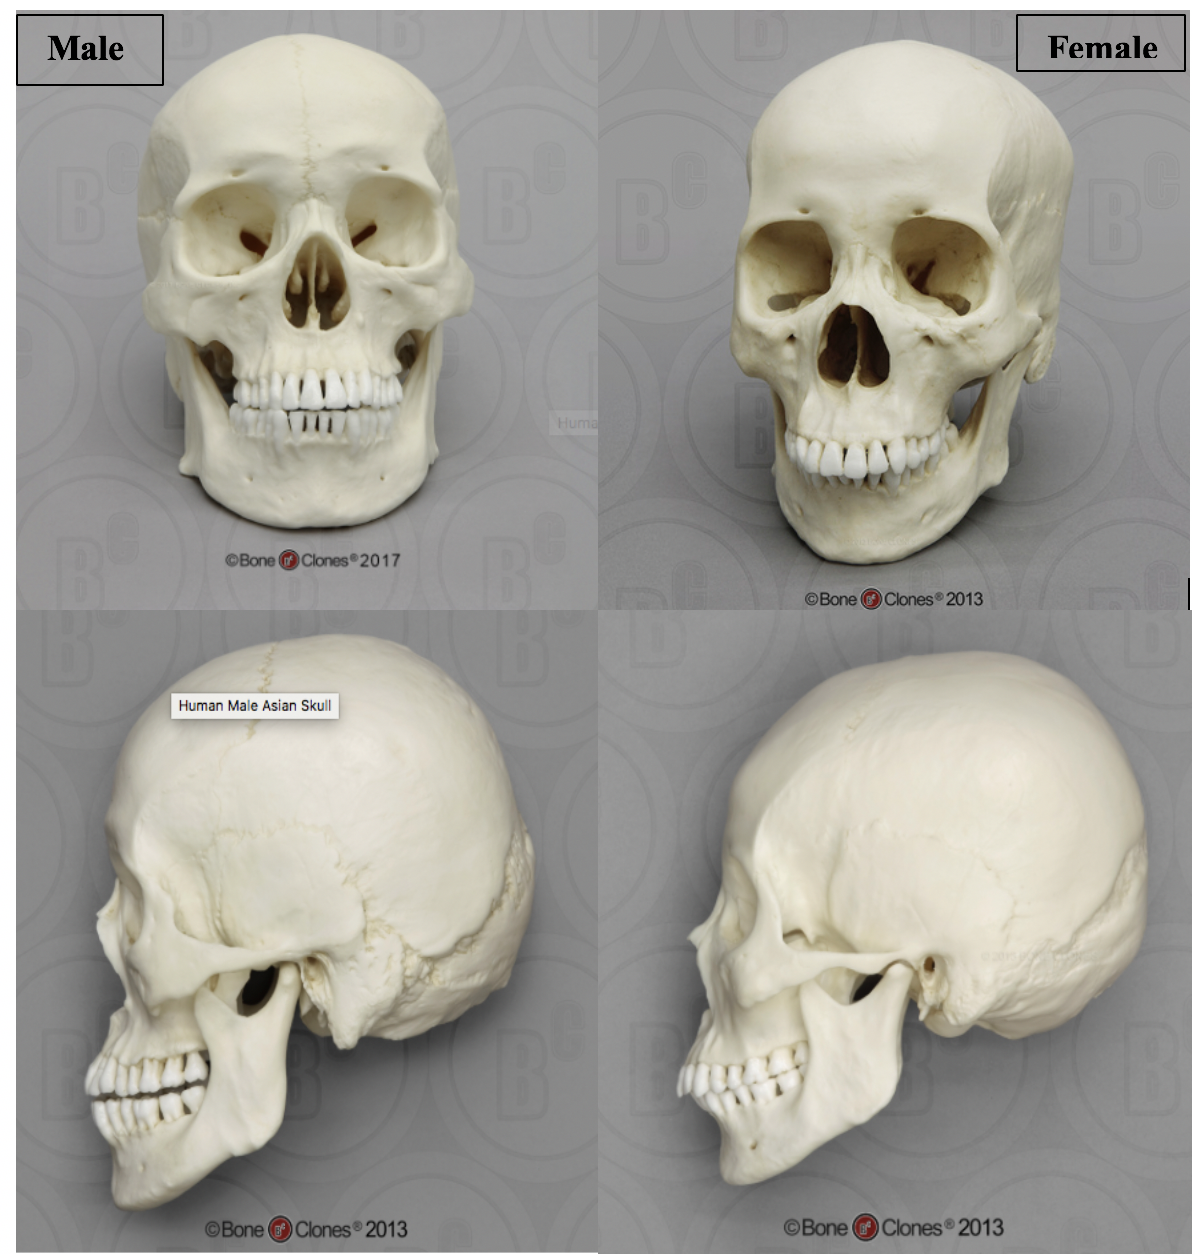
Assessment of biological sex focuses on differences in both morphological (form or structure) and metric (measured) traits in individuals. When assessing morphological traits, the skull and the pelvis are the most commonly referenced areas of the skeleton. These differences are related to sexual dimorphism usually varying in the amount of robusticity seen between males and females. Robusticity deals with strength and size; it is frequently used as a term to describe a large size or thickness. In general, males will show a greater degree of robusticity than females. For example, the length and width of the mastoid process, a bony projection located behind the opening for the ear, is typically larger in males. The mastoid process is an attachment point for muscles of the neck, and this bony projection tends to be wider and longer in males. In general, cranial features tend to be more robust in males (Figure 16.10).
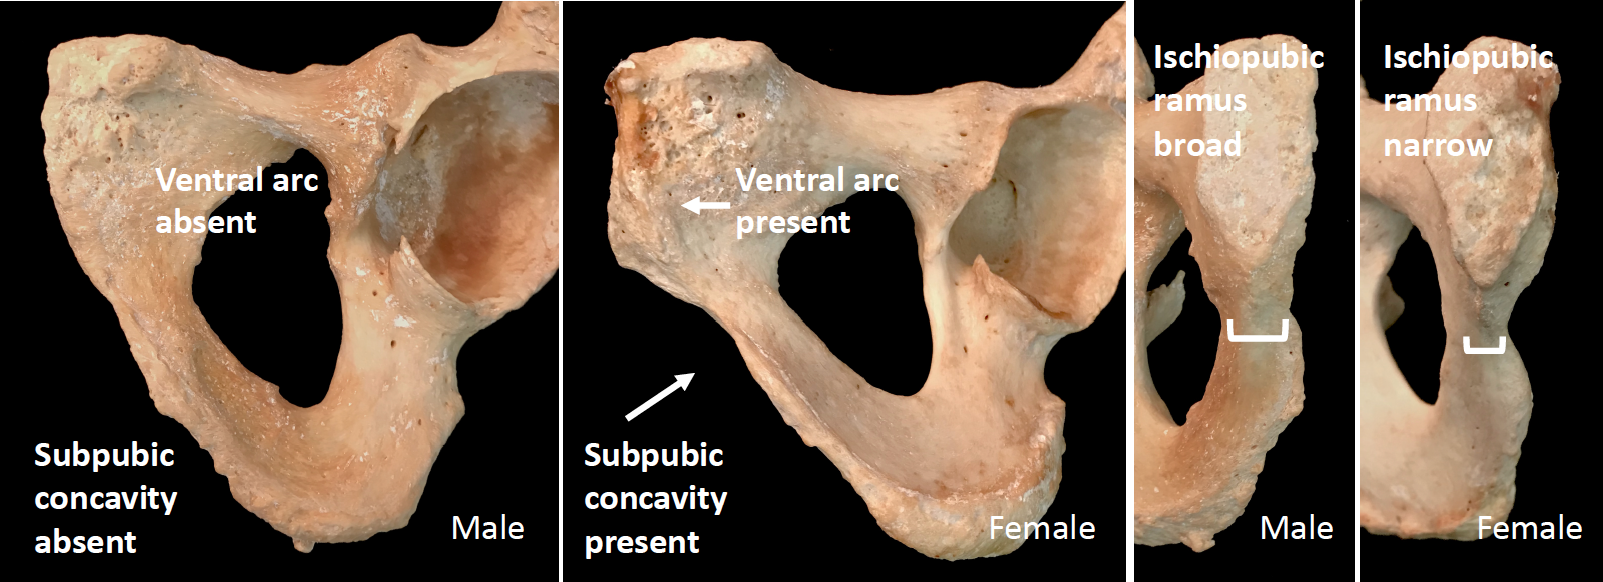
When considering the pelvis, the features associated with the ability to give birth help distinguish females from males. During puberty, estrogen causes a widening of the female pelvis to allow for the passage of a baby. Several studies have identified specific features or bony landmarks associated with the widening of the hips, and this section will discuss one such method. The Phenice Method (Phenice 1969) is traditionally the most common reference used to assess morphological characteristics associated with sex. The Phenice Method specifically looks at the presence or absence of (1) a ventral arc, (2) the presence or absence of a subpubic concavity, and (3) the width of the medial aspect of the ischiopubic ramus (Figure 16.11). When present, the ventral arc, a ridge of bone located on the ventral surface of the pubic bone, is indicative of female remains. Likewise the presence of a subpubic concavity and a narrow medial aspect of the ischiopubic ramus is associated with a female sex estimation. Assessments of these features, as well as those of the skull (when both the pelvis and skull are present), are combined for an overall estimation of sex.
Metric analyses are also used in the estimation of sex. Measurements taken from every region of the body can contribute to estimating sex through statistical approaches that assign a predictive value of sex. These approaches can include multiple measurements from several skeletal elements in what is called multivariate (multiple variables) statistics. Other approaches consider a single measurement, such as the diameter of the head of the femur, of a specific element in a univariate (single variable) analysis (Berg 2017, 152–156).
It is important to note that, although forensic anthropologists usually begin assessment of biological profile with biological sex, there is one major instance in which this is not appropriate. The case of two individuals found in California, on July 8, 1979, is one example that demonstrates the effect age has on the estimation of sex. The identities of the two individuals were unknown; therefore, law enforcement sent them to a lab for identification. A skeletal analysis determined that the remains represented one adolescent male and one adolescent female, both younger than 18 years of age. This information did not match with any known missing children at the time.
In 2015, the cold case was reanalysed, and DNA samples were extracted. The results indicated that the remains were actually those of two girls who went missing in 1978. The girls were 15 years old and 14 years old at the time of death. It is clear that the 1979 results were incorrect, but this mistake also provides the opportunity to discuss the limitations of assessing sex from a subadult skeleton.
Assessing sex from the human skeleton is based on biological and genetic traits associated with females and males. These traits are linked to differences in sexual dimorphism and reproductive characteristics between females and males. The link to reproductive characteristics means that most indicators of biological sex do not fully manifest in prepubescent individuals, making estimations of sex unreliable in younger individuals (SWGANTH 2010b). This was the case in the example of the 14-year-old girl. When examined in 1979, her remains were misidentified as male because she had not yet fully developed female pelvic traits.
Sex vs. Gender
Biological sex is a different concept than gender. While biological anthropologists can estimate sex from the skeleton, estimating an individual’s gender would require a greater context because gender is defined culturally rather than biologically. Take, for example, an individual who identifies as transgender. This individual has a gender identity that is different from their biological sex. The gender identity of any individual depends on factors related to self-identification, situation or context, and cultural factors. While in the U.S. we have historically thought of sex and gender as binary concepts (male or female), many cultures throughout the world recognize several possible gender identities. In this sense, gender is seen as a continuous or fluid variable rather than a fixed one.
Historically, forensic anthropologists have used a binary construct to categorize human skeletal remains as either male or female (with the accompanying categories of probable male, probable female, and indeterminate). In the case of transgender and gender nonconforming individuals, the binary approach to sex assessment may delay or hinder identification efforts (Buchanan 2014; Schall, Rogers, and Deschamps-Braly 2020; Tallman, Kincer, and Plemons 2021). As such, many forensic anthropologists have begun to address the inherent problems associated with a binary approach to sex identification and to explore ways of assessing social identity and self-identified gender using skeletal remains and forensic context.
For the duration of this section, the term transgender refers to individuals whose gender identity differs from the sex assigned at birth (Schall, Rogers, and Deschamps-Braly 2020:2). Transgender individuals transition from one gender binary to another, such as male-to-female (MTF) or female-to-male (FTM). While many of the gender-affirming procedures available to trans and gender-nonconforming individuals are focused on soft tissue modifications (e.g., breast augmentation, genital reconstruction, hormone therapies, etc.), there are a number of gender-affirmation surgeries that do leave a permanent record on the skeleton. Generally speaking, FTM transgender people are reported to undergo fewer surgical procedures than do MTF transgender people (Buchanan 2014). The discussion below focuses on Facial Feminization Surgery (FFS), which leaves a permanent record on the human skeleton that may be used to help make an identification.
FFS refers to a combination of procedures focused on sexually dimorphic features of the face, with the intent of transforming typically male facial features into more feminine forms. Facial Feminization Surgery procedures were developed by Dr. Douglas Ousterhout, a San Francisco based cranio-maxillofacial surgeon, in the mid-1980s (Schall, Rogers, and Deschamps-Braly 2020:2). FFS can include one or a combination of the following: hairline lowering, forehead reduction and contouring, brow lift, reduction rhinoplasty, cheek enhancement, lip lift, lip filling, chin contouring, jaw contouring, and/or tracheal shave (Buchanan 2014; Schall, Rogers, and Deschamps-Braly 2020:2). Of the procedures outlined previously, four are known to directly affect the facial skeleton: forehead contouring, rhinoplasty, chin contouring, and jaw contouring (Buchanan 2014; Schall, Rogers, and Deschamps-Braly 2020:2).
Because FFS procedures have been widely documented in the medical (and more recently the forensic anthropological) literature, there are a number of indicators that a forensic anthropologist can use to make more informed evaluations of gender, including evidence of bone remodeling in sexually dimorphic regions of the skull (e.g., forehead, chin, jawline), as well as the presence of plates, pins, or other surgical hardware that may be evidence of FFS (Buchanan 2014; Schall, Rogers, and Deschamps-Braly 2020; Tallman, Kincer, and Plemons 2021). Additionally, some forensic anthropologists suggest cautiously integrating contextual information from the scene, such as personal effects, material evidence, and recovery scene information, into their evaluation of an individual’s social identity (Beatrice and Soler 2016; Birkby, Fenton, and Anderson 2008; Soler and Beatrice 2018; Soler Et al. 2019; Tallman, Kincer, and Plemons 2021; Winburn, Schoff, and Warren 2016). The ultimate goal of many skeletal analyses is to make a positive identification on a set of unidentified remains.
Assessment of Population Affinity
In an effort to combat the erroneous assumptions tied to the race concept, forensic anthropologists have attempted to reframe this component of the biological profile. The term race is no longer used in casework and teaching. Historically, the word ancestry is and was deemed a more appropriate way to describe an individual’s phenotype. However, in more recent years, forensic anthropologists have begun using the term population affinity, recognizing that we are basing our analysis on the similarities we see based on the reference samples we have available (Winburn and Algee-Hewitt 2021). An important note here is that it is possible to hinder identifications and harm individuals when tools like estimations of population affinity are misapplied, misinterpreted, or misused. For this reason, the field of forensic anthropology has ongoing conversations about the appropriateness of this analysis in the biological profile (Bethard and DiGangi 2020; Stull Et al. 2021).
We use the term population affinity to refer to the variation seen among modern populations—variation that is both genetic and environmentally driven. The word affinity refers to similarities or relationships between individuals. As forensic anthropologists, we compare an unknown individual to multiple reference groups and look for the degree of similarity in observable traits with those groups. As noted previously, population affinity can aid law enforcement in their identification of missing persons or unknown skeletal remains.
Within the field of anthropology, the estimation of population affinity has a contentious history, and early attempts at classification were largely based on the erroneous assumption that an individual’s phenotype (outward appearance) was correlated with their innate intelligence and abilities (see Chapter 14 for a more in-depth discussion of the history of the race concept). The use of the term race is deeply embedded in the social context of the United States. In any other organism/living thing, groups divided according to the biological race concept would be defined as a separate subspecies. The major issue with applying the biological race concept to humans is that there are not enough differences between any two populations to separate on a genetic basis. In other words, biological races do not exist in human populations. However, the concept of race has been perpetuated and upheld by sociocultural constructs of race.
The conundrum for forensic anthropologists is the fact that while races do not exist on a biological level, we still socially recognize and categorize individuals based on their phenotype. Clearly, our phenotype is an important factor in not only how we are viewed by others but also how we identify ourselves. It is also a commonly reported variable. Often labeled as “race,” we are asked to report how we self-identify on school applications, government identification, surveys, census reports, and so forth. It follows then that when a person is reported missing, the information commonly collected by law enforcement and sometimes entered into a missing person’s database includes their age, biological sex, stature, and “race.” Therefore, the more information a forensic anthropologist can provide regarding the individual’s physical characteristics, the more he or she can help to narrow the search.
As an exercise, create a list of all of the women you know who are between the ages of 18 and 24 and approximately 5’ 4” to 5’ 9” tall. You probably have several dozen people on the list. Now, consider how many females you know who are between the ages of 18 and 24, are approximately 5’ 4” to 5’ 9” tall, and are Vietnamese. Your list is going to be significantly shorter. That’s how missing persons searches go as well. The more information you can provide regarding a decedent’s phenotype, the fewer possible matches law enforcement are left to investigate. This is why population affinity has historically been included as a part of the biological profile.
Traditionally, population affinity was accomplished through a visual inspection of morphological variants of the skull (morphoscopics). These methods focused on elements of the facial skeleton, including the nose, eyes, and cheek bones. However, in an effort to reduce subjectivity, nonmetric cranial traits are now assessed within a statistical framework to help anthropologists better interpret their distribution among living populations (Hefner and Linde 2018). Based on the observable traits, a macromorphoscopic analysis will allow the practitioner to create a statistical prediction of geographic origin. In essence, forensic anthropologists are using human variation in the estimation of geographic origin, by referencing documented frequencies of nonmetric skeletal indicators or macromorphoscopic traits.
Population affinity is also assessed through metric analyses. The computer program Fordisc is an anthropological tool used to estimate different components of the biological profile, including ancestry, sex, and stature. When using Fordisc, skeletal measurements are input into the computer software, and the program employs multivariate statistical classification methods, including discriminant function analysis, to generate a statistical prediction for the geographic origin of unknown remains based on the comparison of the unknown to the reference samples in the software program. Fordisc also calculates the likelihood of the prediction being correct, as well as how typical the metric data is for the assigned group.
Estimating Age-at-Death
Estimating age-at-death from the skeleton relies on the measurement of two basic physiological processes: (1) growth and development and (2) degeneration (or aging). From fetal development on, our bones and teeth grow and change at a predictable rate. This provides for relatively accurate age estimates. After our bones and teeth cease to grow and develop, they begin to undergo structural changes, or degeneration, associated with aging. This does not happen at such predictable rates and, therefore, results in less accurate or larger age-range estimations.
During growth and development stages, two primary methods used for estimations of age of subadults (those under the age of 18) are epiphyseal union and dental development. Epiphyseal union (or epiphyseal fusion) refers to the appearance and closure of the epiphyseal plates between the primary centres of growth in a bone and the subsequent centres of growth (see Figure 16.7). Prior to complete union, the cartilaginous area between the primary and secondary centres of growth is also referred to as the growth plates (Schaefer, Black, and Scheuer 2009). Different areas of the skeleton have documented differences in the appearance and closure of epiphyses, making this a reliable method for aging subadult remains (SWGANTH 2013).
As an example of its utility in the identification process, epiphyseal development was used to identify two subadult victims of a fatal fire in Flint, Michigan, in February 2010. The remains represented two young girls, ages three and four. Due to the intensity of the fire, the subadult victims were differentiated from each other through the appearance of the patella, the kneecap. The patella is a bone that develops within the tendon of the quadriceps muscle at the knee joint. The patella begins to form around three to four years of age (Cunningham, Scheuer, and Black 2016, 407–409). In the example above, radiographs of the knees showed the presence of a patella in the four-year-old girl and the absence of a clearly discernible patella in the three-year-old.
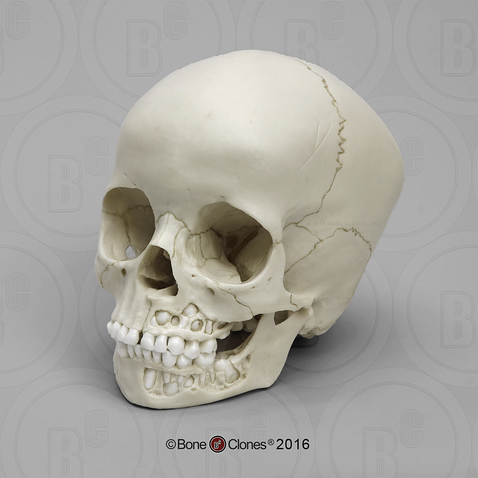
Dental development begins during fetal stages of growth and continues until the complete formation and eruption of the adult third molars (if present). The first set of teeth to appear are called deciduous or baby teeth. Individuals develop a total of 20 deciduous teeth, including incisors, canines, and molars. These are generally replaced by adult dentition as an individual grows (Figure 16.12). A total of 32 teeth are represented in the adult dental arcade, including incisors, canines, premolars, and molars. When dental development is used for age estimations, researchers use both tooth-formation patterns and eruption schedules as determining evidence. For example, the crown of the tooth forms first followed by the formation of the tooth root. During development, an individual can exhibit a partially formed crown or a complete crown with a partially formed root. The teeth generally begin the eruption process once the crown of the tooth is complete. The developmental stages of dentition are one of the most reliable and consistent aging methods for subadults (Langley, Gooding, and Tersigni-Tarrant 2017, 176–177).
Degenerative changes in the skeleton typically begin after 18 years of age, with more prominent changes developing after an individual reaches middle adulthood (commonly defined as after 35 years of age in osteology). These changes are most easily seen around joint surfaces of the pelvis, the cranial vault, and the ribs. In this chapter, we focus on the pubic symphysis surfaces of the pelvis and the sternal ends of the ribs, which show metamorphic changes from young adulthood to older adulthood. The pubic symphysis is a joint that unites the left and right halves of the pelvis. The surface of the pubic symphysis changes during adulthood, beginning as a surface with pronounced ridges (called billowing) and flattening with a more distinct rim to the pubic symphysis as an individual ages. As with all metamorphic age changes, older adults tend to develop lipping around the joint surfaces as well as a breakdown of the joint surfaces. The most commonly used method for aging adult skeletons from the pubic symphysis is the Suchey-Brooks method (Brooks and Suchey 1990; Katz and Suchey 1986). This method divides the changes seen with the pubic symphysis into six phases based on macroscopic age-related changes to the surface. Figure 16.13 provides a visual of the degenerative changes that typically occur on the pubic symphysis.
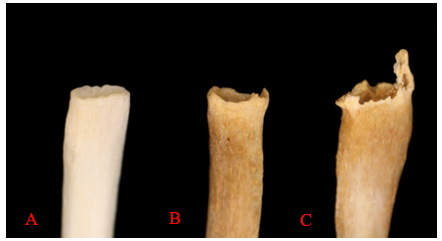
The sternal end of the ribs, the anterior end of the rib that connects via cartilage to the sternum, is also used in age estimations of adults. This method, first developed by M. Y. İşcan and colleagues, considers both the change in shape of the sternal end as well as the quality of the bone (İşcan, Loth, and Wright 1984; İşcan, Loth, and Wright 1985). The sternal end first develops a billowing appearance in young adulthood. The bone typically develops a wider and deeper cupped end as an individual ages. Older adults tend to exhibit bony extensions of the sternal end rim as attaching cartilage ossifies. Figure 16.14 provides a visual of the degenerative changes that typically occur in sternal rib ends.
Estimating Stature
Stature, or height, is one of the most prominently recorded components of the biological profile. Our height is recorded from infancy through adulthood. Doctor’s appointments, driver’s license applications, and sports rosters all typically involve a measure of stature for an individual. As such, it is also a component of the biological profile nearly every individual will have on record. Bioarchaeologists and forensic anthropologists use stature estimation methods to provide a range within which an individual’s biological height would fall. Biological height is a person’s true anatomical height. However, the range created through these estimations is often compared to reported stature, which is typically self-reported and based on an approximation of an individual’s true height (Ousley 1995).
In June 2015, two men were shot and killed in Granite Bay, California, in a double homicide. Investigators were able to locate surveillance camera footage from a gas station where the two victims were spotted in a car with another individual believed to be the perpetrator in the case. The suspect, sitting behind the victims in the car, hung his right arm out of the window as the car drove away. The search for the perpetrator was eventually narrowed down to two suspects. One suspect was 5’ 8” while the other suspect was 6’ 4”, representing almost a foot difference in height reported stature between the two. Forensic anthropologists were given the dimensions of the car (for proportionality of the arm) and were asked to calculate the stature of the suspect in the car from measurements of the suspect’s forearm hanging from the window. Approximate lengths of the bones of the forearm were established from the video footage and used to create a predicted stature range. Stature estimations from skeletal remains typically look at the correlation between the measurements of any individual bone and the overall measurement of body height. In the case above, the length of the right forearm pointed to the taller of the two suspects who was subsequently arrested for the homicide.
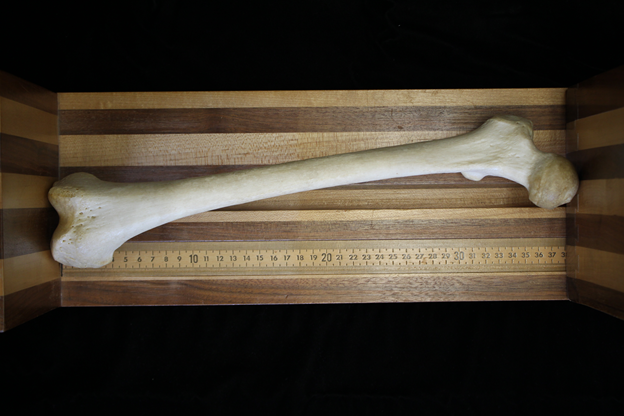
Certain bones, such as the long bones of the leg, contribute more to our overall height than others and can be used with mathematical equations known as regression equations. Regression methods examine the relationship between variables such as height and bone length and use the correlation between the variables to create a prediction interval (or range) for estimated stature. This method for calculating stature is the most commonly used method (SWGANTH 2012). Figure 16.15 shows the measurement of the bicondylar length of the femur for stature estimations.
Identification Using Individualizing Characteristics
One of the most frequently requested analyses within the forensic anthropology laboratory is assistance with the identification of unidentified remains. While all components of a biological profile, as discussed above, can assist law enforcement officers and medical examiners to narrow down the list of potential identifications, a biological profile will not lead to a positive identification. The term positive identification refers to a scientifically validated method of identifying previously unidentified remains. Presumptive identifications, however, are not scientifically validated; rather, they are based on circumstances or scene context. For example, if a decedent is found in a locked home with no evidence of forced entry but the body is no longer visually identifiable, it may be presumed that the remains belong to the homeowner. Hence, a presumptive identification.
The medicolegal system ultimately requires that a positive identification be made in such circumstances, and a presumptive identification is often a good way to narrow down the pool of possibilities. Biological profile information also assists with making a presumptive identification based on an individual’s phenotype in life (e.g., what they looked like). As an example, a forensic anthropologist may establish the following components of a biological profile: white male, between the ages of 35 and 50, approximately 5’ 7” to 5’ 11.” While this seems like a rather specific description of an individual, you can imagine that this description fits dozens, if not hundreds, of people in an urban area. Therefore, law enforcement can use the biological profile information to narrow their pool of possible identifications to include only white males who fit the age and height outlined above. Once a possible match is found, the decedent can be identified using a method of positive identification.
Positive identifications are based on what we refer to as individualizing traits or characteristics, which are traits that are unique at the individual level. For example, brown hair is not an individualizing trait as brown is the most common hair colour in the U.S. But, a specific pattern of dental restorations or surgical implants can be individualizing, because it is unlikely that you will have an exact match on either of these traits when comparing two individuals.
A number of positive methods are available to forensic anthropologists, and for the remainder of this section we will discuss the following methods: comparative medical and dental radiography and identification of surgical implants.
Comparative medical and dental radiography is used to find consistency of traits when comparing antemortem records (medical and dental records taken during life) with images taken postmortem (after death). Comparative medical radiography focuses primarily on features associated with the skeletal system, including trabecular pattern (internal structure of bone that is honeycomb in appearance), bone shape or cortical density (compact outer layer of bone), and evidence of past trauma, skeletal pathology, or skeletal anomalies. Other individualizing traits include the shape of various bones or their features, such as the frontal sinuses (Figure 16.16).
Comparative dental radiography focuses on the number, shape, location, and orientation of dentition and dental restorations in antemortem and postmortem images. While there is not a minimum number of matching traits that need to be identified for an identification to be made, the antemortem and postmortem records should have enough skeletal or dental consistencies to conclude that the records did in fact come from the same individual (SWGANTH 2010a). Consideration should also be given to population-level frequencies of specific skeletal and dental traits. If a trait is particularly common within a given population, it may not be a good trait to utilize for positive identification.
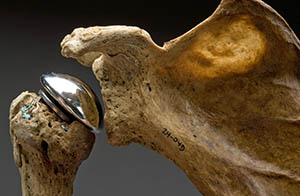
Surgical implants or devices can also be used for identification purposes (Figure 16.17). These implements are sometimes recovered with human remains. One of the ways forensic anthropologists can use surgical implants to assist in decedent identification is by providing a thorough analysis of the implant and noting any identifying information such as serial numbers, manufacturer symbols, and so forth. This information can then sometimes be tracked directly to the manufacturer or the place of surgical intervention, which may be used to identify unknown remains (SWGANTH 2010a).
Special Topic: Trans Doe Task Force
The Trans Doe Task Force (TDTF) is a Trans-led nonprofit organization that investigates cases involving LGBTQ+ missing and murdered persons. The organization specifically focuses on transgender and gender-variant cases, providing connections between law enforcement agencies, medical examiner offices, forensic anthropologists, and forensic genetic genealogists to increase the chances of identification. Additionally, the TDTF curates a data repository of missing, murdered, and unclaimed LGBTQ+ individuals, and they continuously try innovative approaches to identify these individuals, whose lived gender identity may not match their biological sex.
For more information visit transdoetaskforce.org
Trauma Analysis
Types of Trauma
Within the field of anthropology, trauma is defined as an injury to living tissue caused by an extrinsic force or mechanism (Lovell 1997:139). Forensic anthropologists can assist a forensic pathologist by providing an interpretation of the course of events that led to skeletal trauma. Typically, traumatic injury to bone is classified into one of four categories, defined by the trauma mechanism. A trauma mechanism refers to the force that produced the skeletal modification and can be classified as (1) sharp force, (2) blunt force, (3) projectile, or (4) thermal (burning). Each type of trauma, and the characteristic pattern(s) associated with that particular categorization, will be discussed below.
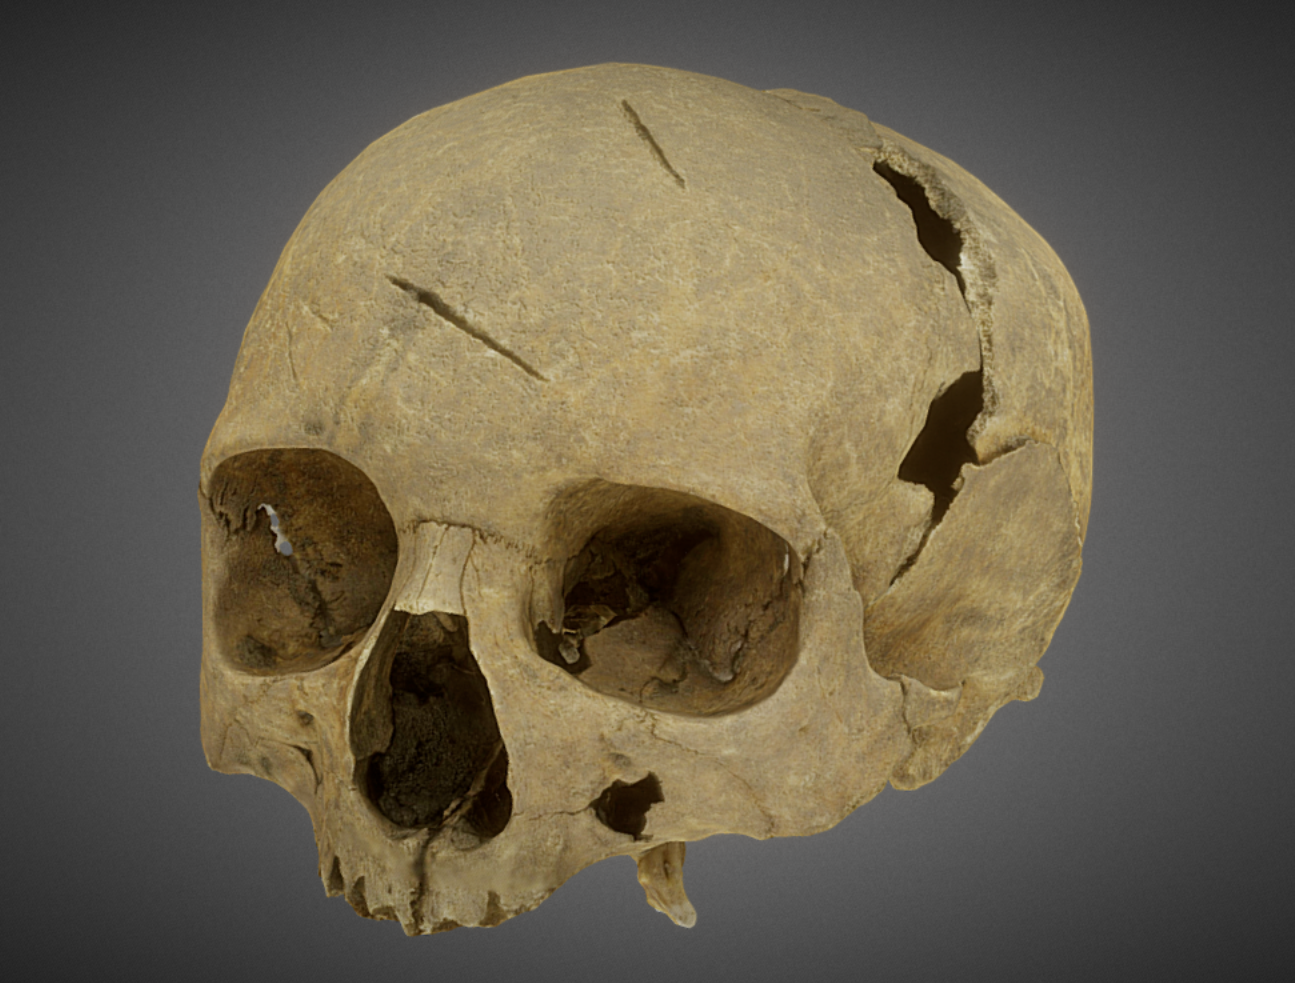
First, let’s consider sharp-force trauma, which is caused by a tool that is edged, pointed, or beveled—for example, a knife, saw, or machete (SWGANTH 2011). The patterns of injury resulting from sharp-force trauma include linear incisions created by a sharp, straight edge; punctures; and chop marks (Figure 16.18; SWGANTH 2011). When observed under a microscope, an anthropologist can often determine what kind of tool created the bone trauma. For example, a power saw cut will be discernible from a manual saw cut.
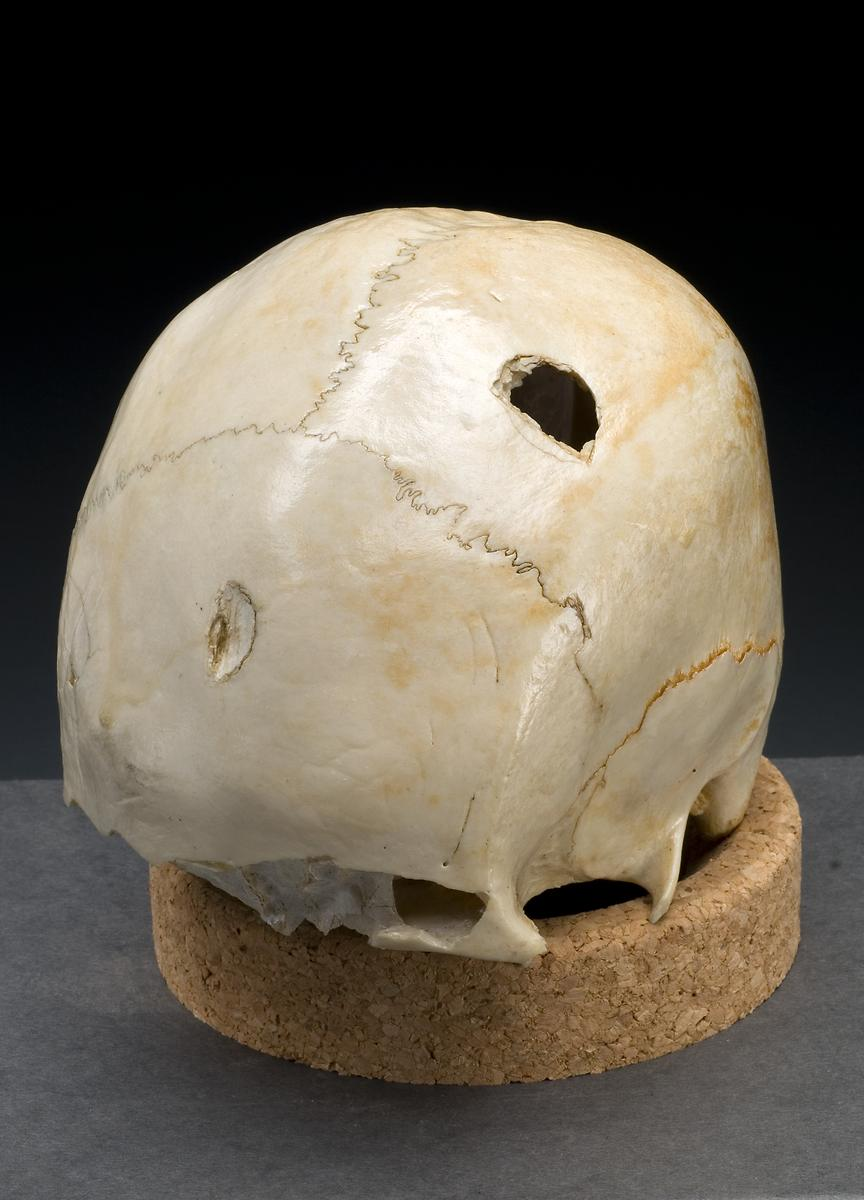
Second, blunt-force trauma is defined as “a relatively low-velocity impact over a relatively large surface area” (Galloway 1999, 5). Blunt-force injuries can result from impacts from clubs, sticks, fists, and so forth. Blunt-force impacts typically leave an injury at the point of impact but can also lead to bending and deformation in other regions of the bone. Depressions, fractures, and deformation at and around the site of impact are all characteristics of blunt-force trauma (Figure 16.19). As with sharp-force trauma, an anthropologist attempts to interpret blunt-force injuries, providing information pertaining to the type of tool used, the direction of impact, the sequence of impacts, if more than one, and the amount of force applied.
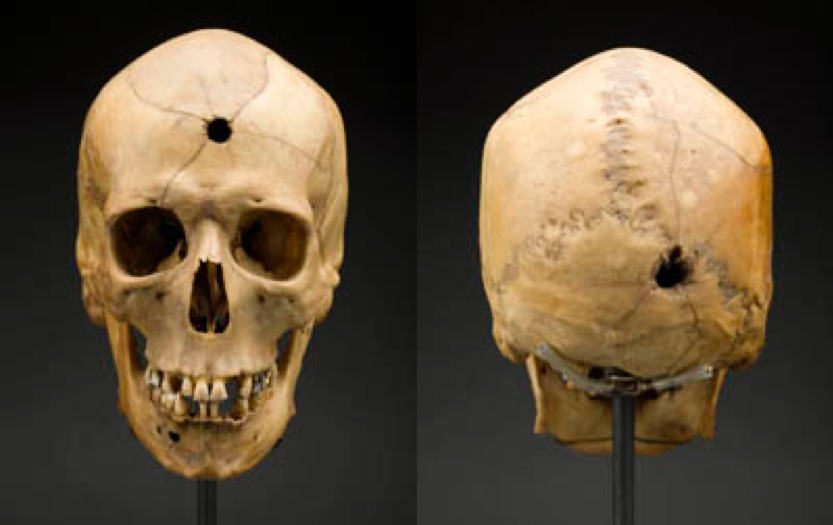
Third, projectile trauma refers to high-velocity trauma, typically affecting a small surface area (Galloway 1999, 6). Projectile trauma results from fast-moving objects such as bullets or shrapnel. It is typically characterized by penetrating defects or embedded materials (Figure 16.20). When interpreting injuries resulting from projectile trauma, an anthropologist can often offer information pertaining to the type of weapon used (e.g., rifle vs. handgun), relative size of the bullet (but not the calibre of the bullet), the direction the projectile was traveling, and the sequence of injuries if there are multiple present.
Finally, thermal trauma is a bone alteration that results from bone exposure to extreme heat. Thermal trauma can result in cases of house or car fires, intentional disposal of a body in cases of homicidal violence, plane crashes, and so on. Thermal trauma is most often characterized by colour changes to bone, ranging from yellow to black (charred) or white (calcined). Other bone alterations characteristic of thermal trauma include delamination (flaking or layering due to bone failure), shrinkage, fractures, and heat-specific burn patterning. When interpreting injuries resulting from thermal damage, an anthropologist can differentiate between thermal fractures and fractures that occurred before heat exposure, thereby contributing to the interpretation of burn patterning (e.g., was the individual bound or in a flexed position prior to the fire?).
While there are characteristic patterns associated with the four categories of bone trauma, it is also important to note that these bone alterations do not always occur independently of different trauma types. An individual’s skeleton may present with multiple different types of trauma, such as a projectile wound and thermal trauma. Therefore, it is important that the anthropologist recognize the different types of trauma and interpret them appropriately.
Timing of Injury
Another important component of any anthropological trauma analysis is the determination of the timing of injury (e.g., when did the injury occur). Timing of injury is traditionally split into one of three categories: antemortem (before death), perimortem (at or around the time of death), and postmortem (after death). This classification system differs slightly from the classification system used by the pathologist because it specifically references the qualities of bone tissue and bone response to external forces. Therefore, the perimortem interval (at or around the time of death) means that the bone is still fresh and has what is referred to as a green bone response, which can extend past death by several weeks or even months. For example, in cold or freezing temperatures a body can be preserved for extended periods of time, increasing the perimortem interval, while in desert climates decomposition is accelerated, thereby significantly decreasing the postmortem interval (Galloway 1999, 12). Antemortem injuries (occurring well before death and not related to the death incident) are typically characterized by some level of healing, in the form of a fracture callus or unification of fracture margins. Finally, postmortem injuries (occurring after death, while bone is no longer fresh) are characterized by jagged fracture margins, resulting from a loss of moisture content during the decomposition process (Galloway 1999, 16). In general, all bone traumas should be classified according to the timing of injury, if possible. This information will help the medical examiner or pathologist better understand the circumstances surrounding the decedent’s death, as well as events occurring during life and after the final disposition of the body.
The Role of the Forensic Anthropologist in Trauma Analysis
Within the medicolegal system, forensic anthropologists are often called upon by the medical examiner, forensic pathologist, or coroner to assist with an interpretation of trauma. The forensic anthropologist’s main focus in any trauma analysis is the underlying skeletal system—as well as, sometimes, cartilage. Analysis and interpretation of soft tissue injuries fall within the purview of the medical examiner or pathologist. It is also important to note that the main role of the forensic anthropologist is to provide information pertaining to skeletal injury to assist the medical examiner/pathologist in their final interpretation of injury. Forensic anthropologists do not hypothesize as to the cause of death of an individual. Instead, a forensic anthropologist’s report should include a description of the injury (e.g., trauma mechanism, number of injuries, location, timing of injury); documentation of the injury, which may be utilized in court testimony (e.g., photographs, radiographs, measurements); and, if applicable, a statement as to the condition of the body and state of decomposition, which may be useful for understanding the depositional context (e.g., how long has the body been exposed to the elements; was it moved or in its original location; are any of the alterations to bone due to environmental or faunal exposure instead of intentional human modification).
Taphonomy
What Happened to the Remains After Death?
The majority of the skeletal analysis process revolves around the identity of the deceased individual. However, there is one last, very important question that forensic anthropologists should ask: What happened to the remains after death? Generally speaking, processes that alter the bone after death are referred to as taphonomic changes (refer to Chapter 8 for a discussion regarding taphonomy and the fossil record).
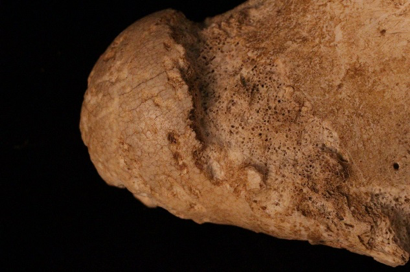
The term taphonomy was originally used to refer to the processes through which organic remains mineralize, also known as fossilization. Within the context of biological anthropology, the term taphonomy is better defined as the study of what happens to human remains after death (Komar and Buikstra 2008). Initial factors affecting a body after death include processes such as decomposition and scavenging by animals. However, taphonomic processes encompass much more than the initial period after death. For example, plant root growth can leach minerals from bone, leaving a distinctive mark. Sunlight can bleach human remains, leaving exposed areas whiter than those that remained buried. Water can wear the surface of the bone until it becomes smooth.
Some taphonomic processes can help a forensic anthropologist estimate the relative amount of time that human remains have been exposed to the elements. For example, root growth through a bone would certainly indicate a body was buried for more than a few days. Forensic anthropologists must be very careful when attempting to estimate time since death based on taphonomic processes because environmental conditions can greatly influence the rate at which taphonomic processes progress. For example, in cold environments, tissue may decay slower than in warm, moist environments.
Forensic anthropologists must contend with taphonomic processes that affect the preservation of bones. For example, high acidity in the soil can break down human bone to the point of crumbling. In addition, when noting trauma, they must be very careful not to confuse postmortem (after death) bone damage with trauma.
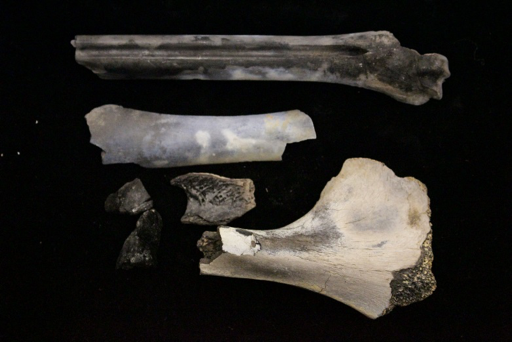
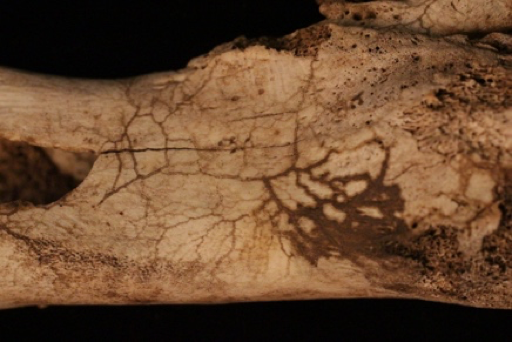
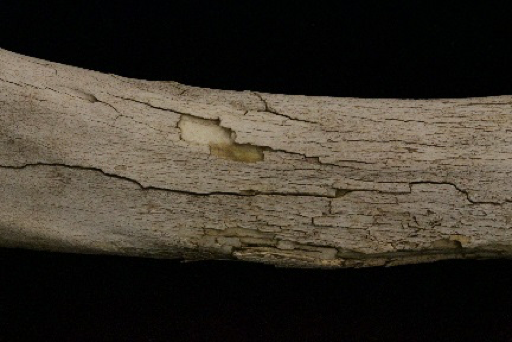
|
Taphonomic Process |
Definition |
|
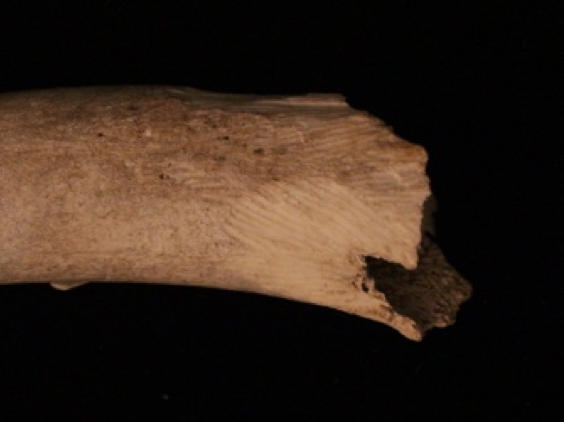
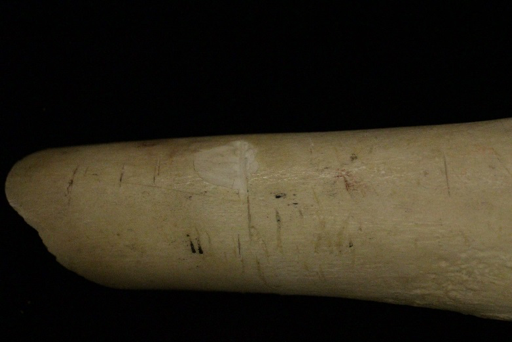
Rodent Gnawing
|
When rodents, such as rats and mice, chew on bone, they leave sets of parallel grooves. The shallow grooves are etched by the rodent’s incisors. |
|
Carnivore Damage
|
Carnivores may leave destructive dental marks on bone. The tooth marks may be visible as pit marks or punctures from the canines, as well as extensive gnawing or chewing of the ends of the bones to retrieve marrow. |
|
Burned Bone
|
Fire causes observable damage to bone. Temperature and the amount of time bone is heated affect the appearance of the bone. Very high temperatures can crack bone and result in white colouration. Colour gradients are visible in between high and lower temperatures, with lower temperatures resulting in black colouration from charring. Cracking can also reveal information about the directionality of the burn. |
|
Root Etching
|
Plant roots can etch the outer surface of bone, leaving grooves where the roots attached as they leached nutrients. During this process, the plant’s roots secrete acid that breaks down the surface of the bone.
|
|
Weathering
|
Many different environmental conditions affect bone. River transport can smooth the surface of the bone due to water abrasion. Sunlight can bleach the exposed surface of bone. Dry and wet environments or the mixture of both types of environments can cause cracking and exfoliation of the surface. Burial in different types of soil can cause discolouration, and exposure can cause degreasing. |
|
Cut Marks
|
Humans may alter bone by cutting, scraping, or sawing it directly or in the process of removing tissue. The groove pattern—that is, the depth and width of the cuts—can help identify the tool used in the cutting process. |
Dig Deeper: Modern Forensic Technologies
In recent years, the forensics community has greatly benefited from the introduction of new technologies, helping strengthen the precision and speed of discoveries and advancements in the field. With recent developments in forensic anthropology, such as 3D scanning technologies, virtual reconstruction, and AI-assisted DNA analysis being integrated into traditional methods, there have been notable changes in how experts investigate human remains.
Artificial intelligence
In recent years, Artificial intelligence (AI) has shown itself to be a valuable tool within forensic anthropology. Aiding forensic experts and toxicologists with complex tasks, the limitations of traditional autopsies can be addressed with the help of AI. By automating and enhancing key investigative processes such as searching for microscopic changes in the human body to determine the cause of death or a person’s life conditions, AI has the potential to enhance the efficiency of forensic processes significantly. It facilitates the detection of microscopic bodily changes to determine the cause of death or living conditions, compares evidence against databases for weapon identification and blood spatter analysis, and reduces manual workload. AI also enables the electronic storage of biometric data–such as facial features, retinal patterns, and fingerprints–for more accurate identity verification. Additionally, AI-powered microscopy enhances the detection of biological traces on complex surfaces, while blood biomarker analysis allows for more precise estimations of time of death (Wankhade Et al., 2022).
While AI holds great promise for the future of forensic medicine, a significant challenge remains: sourcing high-quality data to train the algorithms effectively. One of the more recent AI technologies making waves in the forensic anthropology sector is a new automated AI algorithm called the Convolutional Neural Network (CNN). As described by researchers in Switzerland’s national medical journal Healthcare, CNN is a Deep Learning algorithm that allows for the detection of microscopic skull damage from CT scans or soft-tissue predictions of a face based on the skull information provided (Thurzo Et al., 2021). While there are many advantages to using the CNN, the algorithm can be subject to biases in the same way human forensic experts can, as its assessment and pattern recognition of skulls and skeletons depend on the source data initially used for its AI training (2021).
3D Modeling
Identifying complex trauma to bones–such as distinguishing heat fractures following blunt force trauma–remains a significant challenge in forensic anthropology. This is particularly true for irregular skeletal structures like the pelvis, where overlapping trauma types can be difficult to differentiate, leading to these bones often being understudied. A 2024 study done by researchers from the University of Alberta in collaboration with the Michigan State Police explores the use of 3D laser scans and modelling technology to provide a highly detailed analysis of irregular bones with trauma. The study aimed to better distinguish peri-mortem trauma (trauma occurring around the time of death) from post-mortem heat alterations and improve the forensic analysis accuracy of such cases (Friedlander Et al., 2024). The use of 3D laser scans and modelling technology provides very clear, detailed, and coloured scans of bones, showing distinctions between the characteristics of the fractures. Blunt force and sharp force trauma produce a colour gradient on the 3D model that is more gradual and irregular, while heat fractures are more neat and characterized by little colour variation on the 3D models (2024). Other conclusions were also drawn from the study, such as the differences in trauma on fresh bones and bones that have been exposed to the elements for longer. An example of this is the interstitial fluid and collagen fibrils in fresh bones absorbing force, causing more long and jagged fracture lines, as opposed to a brittle fracture that older bones may exhibit (2024).
Overall, the integration of 3D modeling technology offers a reproducible and highly detailed approach for analyzing trauma in anatomically complex and historically understudied skeletal regions. The practicality of this advancement is further emphasized by the researchers, who note that “in many instances, scanned 3D models can be 3D printed for handheld representation of the model without damaging or overhandling the remains” (2024, p. 2). By enhancing the ability to differentiate between various types of trauma and allowing for more convenient and risk-averse methods of research, this technology significantly improves the accuracy and reliability of forensic interpretations.
Ethics and Human Rights
Working with human remains requires a great deal of consideration and respect for the dead. Forensic anthropologists have to think about the ethics of our use of human remains for scientific purposes. How do we conduct casework in the most respectable manner possible? While there are a wide range of ethical considerations to consider when contemplating a career in forensic anthropology, this chapter will focus on two major categories: working with human remains and acting as an expert within the medicolegal system.
Working with Human Remains
Forensic anthropologists work with human remains in a number of contexts, including casework, excavation, research, and teaching. When working with human remains, it is always important to use proper handling techniques. To prevent damage to skeletal remains, bones should be handled over padded surfaces. Skulls should never be picked up by placing fingers in the eye orbits, foramen magnum (hole at the base of the skull for entry of the spinal cord), or through the zygomatic arches (cheekbones). Human remains, whether related to casework, fieldwork, donated skeletal collections, or research, were once living human beings. It is important to always bear in mind that work with remains should be ingrained with respect for the individual and their relatives. In addition to fieldwork, casework, and teaching, anthropologists are often invited to work with remains that come from a bioarchaeological context or from a human rights violation. While this discussion of ethics is not comprehensive, two case examples will be provided below in which an anthropologist must consider the ethical standards outlined above.
Modern Human Rights Violations
Forensic anthropologists may also be called to participate in criminal investigations involving human rights violations. Anthropological investigations may include assistance with identifications, determination of the number of victims, and trauma analyses. In this role, forensic anthropologists play an integral part in promoting human rights, preventing future human rights violations, and providing the evidence necessary to prosecute those responsible for past events. A few ethical considerations for the forensic anthropologist involved in human rights violations include the use of appropriate standards of identification, presenting reliable and unbiased testimony, and maintaining preservation of evidence. For a more comprehensive history of forensic anthropological contributions to human rights violations investigations (see Ubelaker 2018).
Acting as an Expert in the Medicolegal System
In addition to the ethical considerations involved in working with human skeletal remains, forensic anthropologists must abide by ethical standards when they act as experts within the medicolegal system. The role of the forensic anthropologist within the medicolegal system is primarily to provide information to the medical examiner or coroner that will aid in the identification process or determination of cause and manner of death. Forensic anthropologists also may be called to testify in a court of law. In this capacity, forensic anthropologists should always abide by a series of ethical guidelines that pertain to their interpretation, presentation, and preservation of evidence used in criminal investigations. First and foremost, practitioners should never misrepresent their training or education. When appropriate, outside opinions and assistance in casework should be requested (e.g., consulting a radiologist for radiological examinations or odontologist for dental exams). The best interest of the decedent should always take precedence. All casework should be conducted in an unbiased way, and financial compensation should never be accepted as it can act as an incentive to take a biased stance regarding casework. All anthropological findings should be kept confidential, and release of information is best done by the medical examiner or coroner. Finally, while upholding personal ethical standards, forensic anthropologists are also expected to report any perceived ethical violations committed by their peers.
Ethical standards for the field of forensic anthropology are outlined by the Organization of Scientific Area Committees (OSAC) for Forensic Science, administered by the National Institute of Standards and Technology (NIST). OSAC and NIST recently began an initiative to develop standards that would strengthen the practice of forensic science both in the United States and internationally. OSAC’s main objective is to “strengthen the nation’s use of forensic science by facilitating the development of technically sound forensic science standards and by promoting the adoption of those standards by the forensic science community” (NIST n.d.). Additionally, OSAC promotes the establishment of best practices and other guidelines to ensure that forensic science findings and their presentation are reliable and reproducible (NIST 2023).
Special Topic: Native American Graves Protection and Repatriation Act (NAGPRA)
There is a long history in the United States of systematic disenfranchisement of Native American people, including lack of respect for tribal sovereignty. This includes the egregious treatment of Native American human remains. Over several centuries, thousands of Native American remains were removed from tribal lands and held at institutions in the United States, such as museums and universities.
In 1990, a landmark human rights federal law, the Native American Graves Protection and Repatriation Act (NAGPRA), spurred change in the professional standards and practice of biological anthropology and archaeology. NAGPRA established a legal avenue to provide protection for and repatriation of Native American remains, cultural items, and sacred objects removed from Federal or tribal lands to Native American lineal descendants and tribes, and Native Hawaiian organizations. Human remains and associated artifacts, curated in museum collections and federally funded institutions, are subject to three primary provisions outlined by the NAGPRA statute: (1) protection for Native graves on federal and private land; (2) recognition of tribal authority on such lands; and (3) the requirement that all Native skeletal remains and associated artifacts be inventoried and culturally affiliated groups be consulted concerning decisions related to ownership and final disposition (Rose, Green, and Green 1996). NAGPRA legislation was enacted to ensure ethical consideration and treatment of Native remains and to improve dialogue between scientists and Native groups.
- For more information about NAGPRA, visit the Bureau of Reclamation NAGPRA website
- To read the text of the law, visit the US Congress NAGPRA law website.
- For further discussion of NAGPRA history, please see TRACES: An Open Invitation to Archaeology open textbook website
Becoming a Forensic Anthropologist
What does it take to be a forensic anthropologist? Forensic anthropologists are first and foremost anthropologists. While many forensic anthropologists have an undergraduate degree in anthropology, they may also major in biology, criminal justice, pre-law, pre-med, and many other related fields. Practicing forensic anthropologists typically have an advanced degree, either a Master’s or Doctoral degree in Anthropology. Additional training and experience in archaeology, the medico-legal system, rules of evidence, and expert witness testimony are also common. Practicing forensic anthropologists are also encouraged to be board-certified through the American Board of Forensic Anthropology (ABFA). Learn more about the field and educational opportunities on the ABFA website: https://www.theabfa.org/coursework.
Summary
As a subfield of biological anthropology, forensic anthropology encompasses a wide range of methods used to better understand human remains, whether from the present or the past. Through skeletal analysis, forensic anthropologists approach the study of the deceased from multiple perspectives. For instance, they may begin by identifying whether bones are human or animal, determining whether they are modern or archaeological, and assessing whether the remains were buried alone or as part of a larger assemblage. These initial steps provide a foundation for interpreting what the remains represent.
Once a clearer understanding of the remains is established, forensic anthropologists can construct a biological profile of the individual. This process involves estimating biological sex, population affinity, age at death, and stature, as well as examining unique or individualizing features. Together, these elements allow anthropologists to build a more complete picture of the deceased.
Another central responsibility of forensic anthropologists is investigating how the individual died. Trauma analysis plays a key role in this process: Was the person affected by sharp force, blunt force, projectile injuries, or thermal damage? Determining the timing of injuries (whether they occurred before, at, or after death) along with analyzing what happened to the remains afterward, helps anthropologists understand both the cause and context of death. Taphonomic changes provide additional insight into the circumstances surrounding an individual’s final moments.
Working with human remains requires careful consideration and profound respect for the deceased. For this reason, strict methods and ethical guidelines are integral to the profession. Proper handling techniques ensure that human remains are treated with dignity, while ethical standards guide anthropologists in their dual role within both medical and legal systems. Because their expertise can influence the interpretation and presentation of evidence in criminal investigations, forensic anthropologists must adhere to ethical principles. These standards are outlined by the Organization of Scientific Area Committees (OSAC) for Forensic Science, administered by the National Institute of Standards and Technology (NIST).
Review Questions
- What is forensic anthropology? What are the seven primary steps involved in a skeletal analysis?
- What are the major components of a biological profile? Why are forensic anthropologists often-tasked with creating biological profiles for unknown individuals?
- What are the four major types of skeletal trauma?
- What is taphonomy, and why is an understanding of taphonomy often critical in forensic anthropology analyses?
- What are some of the ethical considerations faced by forensic anthropologists?
For Further Exploration
The American Board of Forensic Anthropology (ABFA)
The American Academy of Forensic Sciences (AAFS)
The Organization of Scientific Area Committees for Forensic Science (OSAC)
References
Adams, Bradley J., and Lyle W. Konigsberg, eds. 2008. Recovery, Analysis, and Identification of Commingled Remains. Totowa, NJ: Humana Press.
Beatrice, Jared S., and Angela Soler. 2016. “Skeletal Indicators of Stress: A Component of the Biocultural Profile of Undocumented Migrants in Southern Arizona.” Journal of Forensic Sciences 61 (5): 1164–1172.
Berg, Gregory E. 2017. “Sex Estimation of Unknown Human Skeletal Remains.” In Forensic Anthropology: A Comprehensive Introduction, Second Edition, edited by Natalie R. Langley and MariaTeresa A. Tersigni-Tarrant, 143–159. Boca Raton, FL: CRC Press.
Bethard, Jonathan D., and Elizabeth A. DiGangi. 2020. “Letter to the Editor—Moving Beyond a Lost Cause: Forensic Anthropology and Ancestry Estimates in the United States.” Journal of Forensic Sciences 65 (5): 1791–1792.
Birkby, Walter H., Todd W. Fenton, and Bruce E. Anderson. 2008. “Identifying Southwest Hispanics Using Nonmetric Traits and the Cultural Profile.” Journal of Forensic Sciences 53 (1): 29–33.
Blatt, Samantha, Amy Michael, and Lisa Bright. Forthcoming. “Bioarchaeology: Interpreting Human Behavior from Skeletal Remains.” In TRACES: An Open Invitation to Archaeology. https://textbooks.whatcom.edu/tracesarchaeology/.
Brooks, S., and J. M. Suchey. 1990. “Skeletal Age Determination Based on the Os Pubis: A Comparison of the Acsádi-Nemeskéri and Suchey-Brooks Methods.” Human Evolution 5 (3): 227–238.
Buchanan, Shelby. 2014. “Bone Modification in Male to Female Transgender Surgeries: Considerations for the Forensic Anthropologist.” MA thesis, Department of Geography and Anthropology, Louisiana State University, Baton Rouge.
Cunningham, Craig, Louise Scheuer, and Sue Black. 2016. Developmental Juvenile Osteology, Second Edition. London: Elsevier Academic Press.
Friedlander, H., Adeeb, S., Correia, P. M., Stone, D., & Brooks‐Lim, E. (2024). An innovative way to use 3d modeling on burnt bone to differentiate heat fractures from blunt and sharp force trauma. WIREs Forensic Science, 6(5), 1–18. https://doi.org/10.1002/wfs2.1525
Galloway, Alison, ed. 1999. Broken Bones: Anthropological Analysis of Blunt Force Trauma. Springfield, IL: Charles C. Thomas Publisher, LTD.
Hefner, Joseph T., and Kandus C. Linde. 2018. Atlas of Human Cranial Macromorphoscopic Traits. San Diego: Academic Press.
İşcan, M. Y., S. R. Loth, and R. K. Wright. 1984. “Age Estimation from the Rib by Phase Analysis: White Males.” Journal of Forensic Sciences 29 (4): 1094–1104.
İşcan, M. Y., S. R. Loth, and R. K. Wright. 1985. “Age Estimation from the Rib by Phase Analysis: White Females.” Journal of Forensic Sciences 30 (3): 853–863.Katz, Darryl, and Judy Myers Suchey. 1986. “Age Determination of the Male Os Pubis.” American Journal of Physical Anthropology 69 (4): 427–435.
Komar, Debra A., and Jane E. Buikstra. 2008. Forensic Anthropology: Contemporary Theory and Practice. New York: Oxford University Press.
Langley, Natalie R., Alice F. Gooding, and MariaTeresa Tersigni-Tarrant. 2017. “Age Estimation Methods.” In Forensic Anthropology: A Comprehensive Introduction, Second Edition, edited by Natalie R. Langley and MariaTeresa A. Tersigni-Tarrant, 175–191. Boca Raton, FL: CRC Press.
Lovell, Nancy C. 1997. “Trauma Analysis in Paleopathology.” Yearbook of Physical Anthropology 104 (S25): 139–170.
Native American Graves Protection and Repatriation Act (NAGPRA) 1990 (25 U.S. Code 3001 et seq.)
NIST (National Institute of Standards and Technology). N.d. “The Organization of Scientific Area Committees for Forensic Science.” Accessed April 18, 2023. https://www.nist.gov/topics/organization-scientific-area-committees-forensic-science.
Ousley, Stephen. 1995. “Should We Estimate Biological or Forensic Stature?” Journal of Forensic Sciences 40(5): 768–773.
Phenice, T. W. 1969. “A Newly Developed Visual Method of Sexing the Os Pubis.” American Journal of Physical Anthropology 30 (2): 297–302.
Rose, Jerome C., Thomas J. Green, and Victoria D. Green. 1996. “NAGPRA Is Forever: Osteology and the Repatriation of Skeletons.” Annual Review of Anthropology 25: 81–103.
Schaefer, Maureen, Sue Black, and Louise Scheuer. Juvenile Osteology: A Laboratory and Field Manual. 2009. San Diego: Elsevier Academic Press.
Schall, Jenna L., Tracy L. Rogers, and Jordan D. Deschamps-Braly. 2020. “Breaking the Binary: The Identification of Trans-women in Forensic Anthropology.” Forensic Science International 309: 110220. https://doi.org/10.1016/j.forsciint.2020.110220.
Scientific Working Group for Forensic Anthropology (SWGANTH). 2010a. “Personal Identification.” Last modified June 3, 2010. https://www.nist.gov/sites/default/files/documents/2018/03/13/swganth_personal_identification.pdf.
Scientific Working Group for Forensic Anthropology (SWGANTH). 2010b. “Sex Assessment.” Last modified June 3, 2010. https://www.nist.gov/sites/default/files/documents/2018/03/13/swganth_sex_assessment.pdf.
Scientific Working Group for Forensic Anthropology (SWGANTH). 2011. “Trauma Analysis.” Last modified May 27, 2011. https://www.nist.gov/sites/default/files/documents/2018/03/13/swganth_trauma.pdf.
Scientific Working Group for Forensic Anthropology (SWGANTH). 2012. “Stature Estimation.” Last modified August 2, 2012. https://www.nist.gov/sites/default/files/documents/2018/03/13/swganth_stature_estimation.pdf.
Scientific Working Group for Forensic Anthropology (SWGANTH). 2013. “Age Estimation.” Last modified January 22, 2013. https://www.nist.gov/sites/default/files/documents/2018/03/13/swganth_age_estimation.pdf.
Soler, Angela, and Jared S. Beatrice. 2018. “Expanding the Role of Forensic Anthropology in Humanitarian Crisis: An Example from the USA-Mexico Border. In Sociopolitics of Migrant Death and Repatriation: Perspectives from Forensic Science, edited by Krista E. Latham and Alyson J. O’Daniel, 115–128. New York: Springer.
Soler, Angela, Robin Reineke, Jared Beatrice, and Bruce E. Anderson. 2019. “Etched in Bone: Embodied Suffering in the Remains of Undocumented Migrants.” In The Border and Its Bodies: The Embodiment of Risk along the U.S.-México Line, edited by Thomas E. Sheridan and Randall H. McGuire, 173–207. Tucson: University of Arizona Press.
Stull, Kyra E., Eric J. Bartelink, Alexandra R. Klales, Gregory E. Berg, Michael W. Kenyhercz, Erica N. L’Abbé, Matthew C. Go, et al.. 2021. “Commentary on: Bethard JD, DiGangi EA. Letter to the Editor—Moving Beyond a Lost Cause: Forensic Anthropology and Ancestry Estimates in the United States. J Forensic Sci. 2020;65(5):1791–2. doi: 10.1111/1556-4029.14513.” Journal of Forensic Sciences 66 (1): 417–420.
Tallman, Sean D., Caroline D. Kincer, and Eric D. Plemons. 2022. “Centering Transgender Individuals in Forensic Anthropology and Expanding Binary Sex Estimation in Casework and Research.” Special issue, “Diversity and Inclusion,” Forensic Anthropology 5 (2): 161–180.
Tersigni-Tarrant, MariaTeresa A., and Natalie R. Langley. 2017. “Human Osteology.” In Forensic Anthropology: A Comprehensive Introduction, Second Edition, edited by Natalie R. Langley and MariaTeresa A. Tersigni-Tarrant, 81–109. Boca Raton, FL: CRC Press.
Thurzo, A., Kosnáčová, H. S., Kurilová, V., Kosmeľ, S., Beňuš, R., Moravanský, N., Kováč, P., Kuracinová, K. M., Palkovič, M., & Varga, I. (2021). Use of Advanced Artificial Intelligence in Forensic Medicine, Forensic Anthropology and Clinical Anatomy. Healthcare (Basel, Switzerland), 9(11), 1545. https://doi.org/10.3390/healthcare9111545
Ubelaker, Douglas H. 2018. “A History of Forensic Anthropology.” Special issue, “Centennial Anniversary Issue of AJPA,” American Journal of Physical Anthropology 165 (4): 915–923.
Wankhade, T. D., Ingale, S. W., Mohite, P. M., & Bankar, N. J. (2022). Artificial Intelligence in forensic medicine and toxicology: The future of forensic medicine. Cureus. https://doi.org/10.7759/cureus.28376
White, Tim D., and Pieter A. Folkens. 2005. The Human Bone Manual. Burlington, MA: Elsevier Academic Press.
Winburn, Allysha P., and Bridget Algee-Hewitt. 2021. “Evaluating Population Affinity Estimates in Forensic Anthropology: Insights from the Forensic Anthropology Database for Assessing Methods Accuracy (FADAMA).” Journal of Forensic Sciences 66 (4): 1210–1219.
Winburn, Allysha Powanda, Sarah Kiley Schoff, and Michael W. Warren. 2016. “Assemblages of the Dead: Interpreting the Biocultural and Taphonomic Signature of Afro- Cuban Palo Practice in Florida.” Journal of African Diaspora Archaeology and Heritage 5 (1): 1–37.
When males and females of a species have different morphological traits.
A strong, long-term relationship between two individuals.
When males and females of a species have similar morphological traits.
Term that describes the male who lives with a group of females.
A group that consists of multiple adult males, multiple adult females, and their dependent offspring.
Societies in which group composition is flexible, such as chimpanzee and spider monkey societies. Individuals may break up into smaller feeding groups (fission) and combine into larger groups (fusion).
The primate family that includes marmosets and tamarins.
A descriptor for an organism that spends most of its time on the ground.
Keith Chan, Ph.D., Grossmont-Cuyamaca Community College District and MiraCosta College
Student contributors to this chapter: Lily Berruyer, Lyn Loytchenko, and Sarah Cupidio
This chapter is a revision from "Chapter 12: Modern Homo sapiens” by Keith Chan. In Explorations: An Open Invitation to Biological Anthropology, first edition, edited by Beth Shook, Katie Nelson, Kelsie Aguilera, and Lara Braff, which is licensed under CC BY-NC 4.0.
Learning Objectives
- Identify the skeletal and behavioural traits that represent modern Homo sapiens.
- Critically evaluate different types of evidence for the origin of our species in Africa and our expansion around the world.
- Understand how the human lifestyle changed when people transitioned from foraging to agriculture.
- Hypothesize how human evolutionary trends may continue into the future.
The walls of a pink limestone cave in the hillside of Jebel Irhoud jutted out of the otherwise barren landscape of the Moroccan desert (Figure 13.1). Miners had excavated the cave in the 1960s, revealing some fossils. In 2007, a re-excavation of the site became a momentous occasion for science. A fossil cranium unearthed by a team of researchers was barely visible to the untrained eye. Just the fossil’s robust brows were peering out of the rock. This research team from the Max Planck Institute for Evolutionary Anthropology was the latest to explore the ancient human presence in this part of North Africa after a find by miners in 1960. Excavating near the first discovery, the researchers wanted to learn more about how Homo sapiens lived far from East Africa, where we thought our species originated.
The scientists were surprised when they analyzed the cranium, named Irhoud 10, and other fossils. Statistical comparisons with other human crania concluded that the Irhoud face shapes were typical of recent modern humans while the braincases matched ancient modern humans. Based on the findings of other scientists, the team expected these modern Homo sapiens fossils to be around 200,000 years old. Instead, dating revealed that the cranium had been buried for around 315,000 years.
Together, the modern-looking facial dimensions and the older date reshaped the interpretation of our species: modern Homo sapiens. Some key evolutionary changes from the archaic Homo sapiens (described in Chapter 12) to our species today happened 100,000 years earlier than we had thought and across the vast African continent rather than concentrated in its eastern region.
This revelation in the study of modern Homo sapiens is just one of the latest in this continually advancing area of biological anthropology. Researchers today are still discovering amazing fossils and ingenious ways to collect data and test hypotheses about our past. Through the collective work of many scientists, we are building an overall theory of modern human origins.
Defining Modernity
What defines modern Homo sapiens when compared to archaic Homo sapiens? Modern humans, like you and me, have a set of derived traits that are not seen in archaic humans or any other hominin. As with other transitions in hominin evolution, such as increasing brain size and bipedal ability, modern traits do not appear fully formed or all at once. In other words, the first modern Homo sapiens was not just born one day from archaic parents. The traits common to modern Homo sapiens appeared in a mosaic manner: gradually and out of sync with one another. There are two areas to consider when tracking the complex evolution of modern human traits. One is the physical change in the skeleton. The other is behaviour inferred from the size and shape of the cranium and material culture evidence.
Skeletal Traits
The skeleton of modern Homo sapiens is less robust than that of archaic Homo sapiens. In other words, the modern skeleton is gracile, meaning that the structures are thinner and smoother. Differences related to gracility in the cranium are seen in the braincase, the face, and the mandible. There are also broad differences in the rest of the skeleton.
Cranial Traits
Several elements of the braincase differ between modern and archaic Homo sapiens. Overall, the shape is much rounder, or more globular, on a modern skull (Lieberman, McBratney, and Krovitz 2002; Neubauer, Hublin, and Gunz 2018; Pearson 2008; Figure 13.2). You can feel the globularity of your own modern human skull. Feel the height of your forehead with the palm of your hand. Viewed from the side, the tall vertical forehead of a modern Homo sapiens stands out when compared to the sloping archaic version. This is because the frontal lobe of the modern human brain is larger than the one in archaic humans, and the skull has to accommodate the expansion. The vertical forehead reduces a trait that is common to all other hominins: the brow ridge or supraorbital torus. The parietal lobes of the brain and the matching parietal bones on either side of the skull both bulge outward more in modern humans. At the back of the skull, the archaic occipital bun is no longer present. Instead, the occipital region of the modern human cranium has a derived tall and smooth curve, again reflecting the globular brain inside.
The trend of shrinking face size across hominins reaches its extreme with our species as well. The facial bones of a modern Homo sapiens are extremely gracile compared to all other hominins (Lieberman, McBratney, and Krovitz 2002). Continuing a trend in hominin evolution, technological innovations kept reducing the importance of teeth in reproductive success (Lucas 2007). As natural selection favoured smaller and smaller teeth, the surrounding bone holding these teeth also shrank.
Related to smaller teeth, the mandible is also gracile in modern humans when compared to archaic humans and other hominins. Interestingly, our mandibles have pulled back so far from the prognathism of earlier hominins that we gained an extra structure at the most anterior point, called the mental eminence. You know this structure as the chin. At the skeletal level, it resembles an upside-down “T” at the centerline of the mandible (Pearson 2008). Looking back at archaic humans, you will see that they all lack a chin. Instead, their mandibles curve straight back without a forward point. What is the chin for and how did it develop? Flora Gröning and colleagues (2011) found evidence of the chin’s importance by simulating physical forces on computer models of different mandible shapes. Their results showed that the chin acts as structural support to withstand strain on the otherwise gracile mandible.
Postcranial Gracility
The rest of the modern human skeleton is also more gracile than its archaic counterpart. The differences are clear when comparing a modern Homo sapiens with a cold-adapted Neanderthal (Sawyer and Maley 2005), but the trends are still present when comparing modern and archaic humans within Africa (Pearson 2000). Overall, a modern Homo sapiens postcranial skeleton has thinner cortical bone, smoother features, and more slender shapes when compared to archaic Homo sapiens (Figure 13.3). Comparing whole skeletons, modern humans have longer limb proportions relative to the length and width of the torso, giving us lankier outlines.
Why is our skeleton so gracile compared to those of other hominins? Natural selection can drive the gracilization of skeletons in several ways (Lieberman 2015). A slender frame is believed to be adapted for the efficient long-distance running ability that started with Homo erectus. Furthermore, it is argued that slenderness is a genetic adaptation for cooling an active body in hotter climates, which aligns with the ample evidence that Africa was the home continent of our species.
Behavioural Modernity
Aside from physical differences in the skeleton, researchers have also uncovered evidence of behavioural changes associated with increased cultural complexity from archaic to modern humans. How did cultural complexity develop? Two investigations into this question are archaeology and the analysis of reconstructed brains.
Archaeology tells us much about the behavioural complexity of past humans by interpreting the significance of material culture. In terms of advanced culture, items created with an artistic flair, or as decoration, speak of abstract thought processes (Figure 13.4). The demonstration of difficult artistic techniques and technological complexity hints at social learning and cooperation as well. According to paleoanthropologist John Shea (2011), one way to track the complexity of past behaviour through artifacts is by measuring the variety of tools found together. The more types of tools constructed with different techniques and for different purposes, the more modern the behaviour. Researchers are still working on an archaeological way to measure cultural complexity that is useful across time and place.
The interpretation of brain anatomy is another promising approach to studying the evolution of human behaviour. When looking at investigations on this topic in modern Homo sapiens brains, researchers found a weak association between brain size and test-measured intelligence (Pietschnig Et al. 2015). Additionally, they found no association between intelligence and biological sex. These findings mean that there are more significant factors that affect tested intelligence than just brain size. Since the sheer size of the brain is not useful for weighing intelligence within a species, paleoanthropologists are instead investigating the differences in certain brain structures. The differences in organization between modern Homo sapiens brains and archaic Homo sapiens brains may reflect different cognitive priorities that account for modern human culture. As with the archaeological approach, new discoveries will refine what we know about the human brain and apply that knowledge to studying the distant past.
Taken together, the cognitive abilities in modern humans may have translated into an adept use of tools to enhance survival. Researchers Patrick Roberts and Brian A. Stewart (2018) call this concept the generalist-specialist niche: our species is an expert at living in a wide array of environments, with populations culturally specializing in their own particular surroundings. The next section tracks how far around the world these skeletal and behavioural traits have taken us.
First Africa, Then the World
What enabled modern Homo sapiens to expand its range further in 300,000 years than Homo erectus did in 1.5 million years? The key is the set of derived biological traits from the last section. It is theorized that the gracile frame and neurological anatomy allowed modern humans to survive and even flourish in the vastly different environments they encountered. Based on multiple types of evidence, the source of all of these modern humans was Africa. Instead of originating from just one location, evidence shows that modern Homo sapiens evolution occurred in a complex gene flow network across Africa, a concept called African multiregionalism (Scerri Et al. 2018).
This section traces the origin of modern Homo sapiens and the massive expansion of our species across all of the continents (except Antarctica) by 12,000 years ago. While modern Homo sapiens first shared geography with archaic humans, modern humans eventually spread into lands where no human had gone before. Figure 13.5 shows the broad routes that our species took expanding around the world. I encourage you to make your own timeline with the dates in this part to see the overall trends.
Modern Homo sapiens Biology and Culture in Africa
We start with the ample fossil evidence supporting the theory that modern humans originated in Africa during the Middle Pleistocene, having evolved from African archaic Homo sapiens. The earliest dated fossils considered to be modern actually have a mosaic of archaic and modern traits, showing the complex changes from one type to the other. Experts have various names for these transitional fossils, such as Early Modern Homo sapiens or Early Anatomically Modern Humans. However they are labeled, the presence of some modern traits means that they illustrate the origin of the modern type. Three particularly informative sites with fossils of the earliest modern Homo sapiens are Jebel Irhoud, Omo, and Herto.
Recall from the start of the chapter that the most recent finds at Jebel Irhoud are now the oldest dated fossils that exhibit some facial traits of modern Homo sapiens. Besides Irhoud 10, the cranium that was dated to 315,000 years ago (Hublin Et al. 2017; Richter Et al. 2017), there were other fossils found in the same deposit that we now know are from the same time period. In total there are at least five individuals, representing life stages from childhood to adulthood. These fossils form an image of high variation in skeletal traits. For example, the skull named Irhoud 1 has a primitive brow ridge, while Irhoud 2 and Irhoud 10 do not (Figure 13.6). The braincases are lower than what is seen in the modern humans of today but higher than in archaic Homo sapiens. The teeth also have a mix of archaic and modern traits that defy clear categorization into either group.
Research separated by nearly four decades uncovered fossils and artifacts from the Kibish Formation in the Lower Omo Valley in Ethiopia. These Omo Kibish hominins were represented by braincases and fragmented postcranial bones of three individuals found kilometers apart, dating back to around 233,000 years ago (Day 1969; McDougall, Brown, and Fleagle 2005; Vidal Et al. 2022). One interesting finding was the variation in braincase size between the two more-complete specimens: while the individual named Omo I had a more globular dome, Omo II had an archaic-style long and low cranium.
Also in Ethiopia, a team led by Tim White (2003) excavated numerous fossils at Herto. There were fossilized crania of two adults and a child, along with fragments of more individuals. The dates ranged between 160,000 and 154,000 years ago. The skeletal traits and stone-tool assemblage were both intermediate between the archaic and modern types. Features reminiscent of modern humans included a tall braincase and thinner zygomatic (cheek) bones than those of archaic humans (Figure 13.7). Still, some archaic traits persisted in the Herto fossils, such as the supraorbital tori. Statistical analysis by other research teams concluded that at least some cranial measurements fit just within the modern human range (McCarthy and Lucas 2014), favouring categorization with our own species.
The timeline of material culture suggests a long period of relying on similar tools before a noticeable diversification of artifacts types. Researchers label the time of stable technology shared with archaic types the Middle Stone Age, while the subsequent time of diversification in material culture is called the Later Stone Age.
In the Middle Stone Age, the sites of Jebel Irhoud, Omo, and Herto all bore tools of the same flaked style as archaic assemblages, even though they were separated by almost 150,000 years. The consistency in technology may be evidence that behavioural modernity was not so developed. No clear signs of art dating back this far have been found either. Other hypotheses not related to behavioural modernity could explain these observations. The tool set may have been suitable for thriving in Africa without further innovation. Maybe works of art from that time were made with media that deteriorated or perhaps such art was removed by later humans.
Evidence of what Homo sapiens did in Africa from the end of the Middle Stone Age to the Later Stone Age is concentrated in South African cave sites that reveal the complexity of human behaviour at the time. For example, Blombos Cave, located along the present shore of the Cape of Africa facing the Indian Ocean, is notable for having a wide variety of artifacts. The material culture shows that toolmaking and artistry were more complex than previously thought for the Middle Stone Age. In a layer dated to 100,000 years ago, researchers found two intact ochre-processing kits made of abalone shells and grinding stones (Henshilwood Et al. 2011). Marine snail shell beads from 75,000 years ago were also excavated (Figure 13.8; d’Errico Et al. 2005). Together, the evidence shows that the Middle Stone Age occupation at Blombos Cave incorporated resources from a variety of local environments into their culture, from caves (ochre), open land (animal bones and fat), and the sea (abalone and snail shells). This complexity shows a deep knowledge of the region’s resources and their use—not just for survival but also for symbolic purposes.
On the eastern coast of South Africa, Border Cave shows new African cultural developments at the start of the Later Stone Age. Paola Villa and colleagues (2012) identified several changes in technology around 43,000 years ago. Stone-tool production transitioned from a slower process to one that was faster and made many microliths, small and precise stone tools. Changes in decorations were also found across the Later Stone Age transition. Beads were made from a new resource: fragments of ostrich eggs shaped into circular forms resembling present-day breakfast cereal O’s (d’Errico Et al. 2012). These beads show a higher level of altering one’s own surroundings and a move from the natural to the abstract in terms of design.
Expansion into the Middle East and Asia
While modern Homo sapiens lived across Africa, some members eventually left the continent. These pioneers could have used two connections to the Middle East or West Asia. From North Africa, they could have crossed the Sinai Peninsula and moved north to the Levant, or eastern Mediterranean. Finds in that region show an early modern human presence. Other finds support the Southern Dispersal model, with a crossing from East Africa to the southern Arabian Peninsula through the Straits of Bab-el-Mandeb. It is tempting to think of one momentous event in which people stepped off Africa and into the Middle East, never to look back. In reality, there were likely multiple waves of movement producing gene flow back and forth across these regions as the overall range pushed east. The expanding modern human population could have thrived by using resources along the southern coast of the Arabian Peninsula to South Asia, with side routes moving north along rivers. The maximum range of the species then grew across Asia.
Modern Homo sapiens in the Middle East
Geographically, the Middle East is the ideal place for the African modern Homo sapiens population to inhabit upon expanding out of their home continent. In the Eastern Mediterranean coast of the Levant, there is a wealth of skeletal and material culture linked to modern Homo sapiens. Recent discoveries from Saudi Arabia further add to our view of human life just beyond Africa.
The Caves of Mount Carmel in present-day Israel have preserved skeletal remains and artifacts of modern Homo sapiens, the first-known group living outside Africa. The skeletal presence at Misliya Cave is represented by just part of the left upper jaw of one individual, but it is notable for being dated to a very early time, between 194,000 and 177,000 years ago (Hershkovitz Et al. 2018). Later, from 120,000 to 90,000 years ago, fossils of multiple individuals across life stages were found in the caves of Es-Skhul and Qafzeh (Shea and Bar-Yosef 2005). The skeletons had many modern Homo sapiens traits, such as globular crania and more gracile postcranial bones when compared to Neanderthals. Still, there were some archaic traits. For example, the adult male Skhul V also possessed what researchers Daniel Lieberman, Osbjorn Pearson, and Kenneth Mowbray (2000) called marked or clear occipital bunning. Also, compared to later modern humans, the Mount Carmel people were more robust. Skhul V had a particularly impressive brow ridge that was short in height but sharply jutted forward above the eyes (Figure 13.9). The high level of preservation is due to the intentional burial of some of these people. Besides skeletal material, there are signs of artistic or symbolic behaviour. For example, the adult male Skhul V had a boar’s jaw on his chest. Similarly, Qafzeh 11, a juvenile with healed cranial trauma, had an impressive deer antler rack placed over his torso (Figure 13.10; Coqueugniot Et al. 2014). Perforated seashells coloured with ochre, mineral-based pigment, were also found in Qafzeh (Bar-Yosef Mayer, Vandermeersch, and Bar-Yosef 2009).
One remaining question is, what happened to the modern humans of the Levant after 90,000 years ago? Another site attributed to our species did not appear in the region until 47,000 years ago. Competition with Neanderthals may have accounted for the disappearance of modern human occupation since the Neanderthal presence in the Levant lasted longer than the dates of the early modern Homo sapiens. John Shea and Ofer Bar-Yosef (2005) hypothesized that the Mount Carmel modern humans were an initial expansion from Africa that failed. Perhaps they could not succeed due to competition with the Neanderthals who had been there longer and had both cultural and biological adaptations to that environment.
Modern Homo sapiens of China
A long history of paleoanthropology in China has found ample evidence of modern human presence. Four notable sites are the caves at Fuyan, Liujiang, Tianyuan, and Zhoukoudian. In the distant past, these caves would have been at least seasonal shelters that unintentionally preserved evidence of human presence for modern researchers to discover.
At Fuyan Cave in Southern China, paleoanthropologists found 47 adult teeth associated with cave formations dated to between 120,000 and 80,000 years ago (Liu Et al. 2015). It is currently the oldest-known modern human site in China, though other researchers question the validity of the date range (Michel Et al. 2016). The teeth have the small size and gracile features of modern Homo sapiens dentition.
The fossil Liujiang (or Liukiang) hominin (67,000 years ago) has derived traits that classified it as a modern Homo sapiens, though primitive archaic traits were also present. In the skull, which was found nearly complete, the Liujiang hominin had a taller forehead than archaic Homo sapiens but also had an enlarged occipital region (Figure 13.11; Brown 1999; Wu Et al. 2008). Other parts of the skeleton also had a mix of modern and archaic traits: for example, the femur fragments suggested a slender length but with thick bone walls (Woo 1959).
Another Chinese site to describe here is the one that has been studied the longest. In the Zhoukoudian Cave system (Figure 13.12), where Homo erectus and archaic Homo sapiens have also been found, there were three crania of modern Homo sapiens. These crania, which date to between 34,000 and 10,000 years ago, were all more globular than those of archaic humans but still lower and longer than those of later modern humans (Brown 1999; Harvati 2009). When compared to one another, the crania showed significant differences from one another. Comparison of cranial measurements to other populations past and present found no connection with modern East Asians, again showing that human variation was very different from what we see today.
Crossing to Australia
Expansion of the first modern human Asians, still following the coast, eventually entered an area that researchers call Sunda before continuing on to modern Australia. Sunda was a landmass made up of the modern-day Malay Peninsula, Sumatra, Java, and Borneo. Lowered sea levels connected these places with land bridges, making them easier to traverse. Proceeding past Sunda meant navigating Wallacea, the archipelago that includes the Indonesian islands east of Borneo. In the distant past, there were many megafauna, large animals that migrating humans would have used for food and materials (such as utilizing animals’ hides and bones). Further southeast was another landmass called Sahul, which included New Guinea and Australia as one contiguous continent. Based on fossil evidence, this land had never seen hominins or any other primates before modern Homo sapiens arrived. Sites along this path offer clues about how our species handled the new environment to live successfully as foragers.
The skeletal remains at Lake Mungo, land traditionally owned by Mutthi Mutthi, Ngiampaa, and Paakantji peoples, are the oldest known in the continent. The now-dry lake was one of a series located along the southern coast of Australia in New South Wales, far from where the first people entered from the north (Barbetti and Allen 1972; Bowler Et al. 1970). Two individuals dating to around 40,000 years ago show signs of artistic and symbolic behaviour, including intentional burial. The bones of Lake Mungo 1 (LM1), an adult female, were crushed repeatedly, coloured with red ochre, and cremated (Bowler Et al. 1970). Lake Mungo 3 (LM3), a tall, older male with a gracile cranium but robust postcranial bones, had his fingers interlocked over his pelvic region (Brown 2000).
Kow Swamp, within traditional Yorta Yorta land also in southern Australia, contained human crania that looked distinctly different from the ones at Lake Mungo (Durband 2014; Thorne and Macumber 1972). The crania, dated between 9,000 and 20,000 years ago, had extremely robust brow ridges and thick bone walls, but these were paired with globular features on the braincase (Figure 13.13).
While no fossil humans have been found at the Madjedbebe rock shelter in the North Territory of Australia, more than 10,000 artifacts found there show both behavioural modernity and variability (Clarkson Et al. 2017). They include a diverse array of stone tools and different shades of ochre for rock art, including mica-based reflective pigment (similar to glitter). These impressive artifacts are as far back as 56,000 years old, providing the date for the earliest-known presence of humans in Australia.
From the Levant to Europe
The first modern human expansion into Europe occurred after other members of our species settled in East Asia and Australia. As the evidence from the Levant suggests, modern human movement to Europe may have been hampered by the presence of Neanderthals. It is suggested that another obstacle was the colder climate, which was incompatible with the biology of modern Homo sapiens from Africa, as they were adapted to high temperatures and ultraviolet radiation. Still, by 40,000 years ago, modern Homo sapiens had a detectable presence. This time was also the start of the Later Stone Age or Upper Paleolithic, when there was an expansion in cultural complexity. There is a wealth of evidence from this region due to a Western bias in research, the proximity of these findings to Western scientific institutions, and the desire of Western scientists to explore their own past.
In Romania, the site of Peștera cu Oase (Cave of Bones) had the oldest-known remains of modern Homo sapiens in Europe, dated to around 40,000 years ago (Trinkaus Et al. 2003a). Among the bones and teeth of many animals were the fragmented cranium of one person and the mandible of another (the two bones did not fit each other). Both bones have modern human traits similar to the fossils from the Middle East, but they also had Neanderthal traits. Oase 1, the mandible, had a mental eminence but also extremely large molars (Trinkaus Et al. 2003b). This mandible has yielded DNA that surprisingly is equally similar to DNA from present-day Europeans and Asians (Fu Et al. 2015). This means that Oase 1 was not the direct ancestor of modern Europeans. The Oase 2 cranium has the derived traits of reduced brow ridges along with archaic wide zygomatic cheekbones and an occipital bun (Figure 13.14; Rougier Et al. 2007).
Dating to around 26,000 years ago, Předmostí near Přerov in the Czech Republic was a site where people buried over 30 individuals along with many artifacts. Eighteen individuals were found in one mass burial area, a few covered by the scapulae of woolly mammoths (Germonpré, Lázničková-Galetová, and Sablin 2012). The Předmostí crania were more globular than those of archaic humans but tended to be longer and lower than in later modern humans (Figure 13.15; Velemínská Et al. 2008). The height of the face was in line with modern residents of Central Europe. There was also skeletal evidence of dog domestication, such as the presence of dog skulls with shorter snouts than in wild wolves (Germonpré, Lázničková-Galetová, and Sablin Et al. 2012). In total, Předmostí could have been a settlement dependent on mammoths for subsistence and the artificial selection of early domesticated dogs.
The sequence of modern Homo sapiens technological change in the Later Stone Age has been thoroughly dated and labeled by researchers working in Europe. Among them, the Gravettian tradition of 33,000 years to 21,000 years ago is associated with most of the known curvy female figurines, often assumed to be “Venus” figures. Hunting technology also advanced in this time with the first known boomerang, atlatl (spear thrower), and archery. The Magdalenian tradition spread from 17,000 to 12,000 years ago. This culture further expanded on fine bone tool work, including barbed spearheads and fishhooks (Figure 13.16).
Among the many European sites dating to the Later Stone Age, the famous cave art sites deserve mention. Chauvet-Pont-d'Arc Cave in southern France dates to separate Aurignacian occupations 31,000 years ago and 26,000 years ago. Over a hundred art pieces representing 13 animal species are preserved, from commonly depicted deer and horses to rarer rhinos and owls. Another French cave with art is Lascaux, which is several thousand years younger at 17,000 years ago in the Magdalenian period. At this site, there are over 6,000 painted figures on the walls and ceiling (Figure 13.17). Scaffolding and lighting must have been used to make the paintings on the walls and ceiling deep in the cave. Overall, visiting Lascaux as a contemporary must have been an awesome experience: trekking deeper in the cave lit only by torches giving glimpses of animals all around as mysterious sounds echoed through the galleries.
Special Topic: Cannibalism and Culture - Mortuary Practices in Modern Homo sapiens
Within a 2017 publication in the Journal of Archaeological Method and Theory, Saladié and Rodríguez-Hidalgo bring light to traces of early cannibalism in western Eurasia, arguing that context-specific cannibalistic practices were present throughout the Pleistocene and increased notably from the end of the Upper Palaeolithic and onward (Saladié & Rodriguez-Hidalgo, 2017). While early hominins and Neandertals are recognized in this research, the authors highlight the presence of these mortuary practices in a cluster of Homo sapiens sites. More recent research uncovers similar findings that back these claims as well, where human bones in Herto Ethiopia, Maszycka Cave Poland, and Gough’s Cave in the United Kingdom show anthropogenic defleshing and other modifications which have been interpreted as cannibalism (Pobiner, Et al. 2023). These findings suggest that cannibalistic behaviours formed a recurring aspect of modern human behaviour in certain ecological and cultural contexts.
A significant example comes from the Neolithic levels of Fontbrégua Cave in southeastern France, where Paola Villa and colleagues compared clusters of human bones with the remains of wild and domestic animals from the same sediments. The study found that human bodies were butchered, processed, and most likely eaten in a way that parallels animal carcass treatment, including the placement and timing of cut marks, dismemberment sequences, and perimortem fractures to open marrow cavities (Villa, Et al. 1986). As the assemblage comes from a primary depositional context with pristine preservation and careful excavation, the authors suggest that cannibalism is the only satisfactory explanation for the pattern of cut marks and breakage seen on the human bones.
More recent work has furthered this hypothesis for Late Upper Palaeolithic Homo sapiens, especially in Magdalenian contexts. In a 2023 study, researchers combined archeological and genetic evidence from fifty-nine Magdalenian sites, concluding that this specific culture shows an unusually high frequency of cannibalistic cases compared to earlier and later hominin groups; so much so that they identify “primary burial and cannibalism” as the two main mortuary expressions (Marsh & Bello, 2023). Additionally, new analyses from Maszycka Cave in Poland have described cut and broken human bones in patterns consistent with human consumption, reinforcing this cannibalism hypothesis (Marginedas & Saladié, 2025). Together, these studies suggest that for some Magdalenian groups, mortuary cannibalism was a habitual way of disposing of the dead, not just a one-off crisis response. At the same time, researchers emphasize that not every modified skeleton indicates blatant consumption of the dead and that ritual or symbolic perspectives must also be considered. Previously noted in chapter 12, Ullrich’s survey of European mortuary practices presents frequent manipulations of corpses from the Palaeolithic through the Hallstatt period. Said manipulations include cut marks, dismemberment, skull fracturing, and marrow extraction (Ullrich, 2005, p. 258), which Ullrich interprets as cannibalistic rites embedded in cult ceremonies rather than everyday subsistence. In the author’s view, some Palaeolithic groups may have believed that consuming members of their community allowed them to take on the strengths,
abilities, or even mental aspects of their dead member; the act of cannibalism may have functioned as a form of appropriating physical and mental powers rather than simply obtaining calories. With that, Neolithic assemblages show how careful taphonomic work can distinguish cuts linked to interpersonal violence from those associated with systemic butchery (Marginedas & Saladié, 2025). The findings seek to highlight that some Homo sapiens populations combined ritual, mortuary, and nutritional motives when processing human remains.
These past and contemporary findings are significant for future anthropology students as they shed light on biological anthropology methodology and interpretation. Archaeologists are able to distinguish between occasions when humans were handled like any other carcass and times when they were handled in more symbolic ways thanks to factors like cut mark orientation, the timing of bone breakage, and direct comparison with animal remains. Readers interested in exploring this topic further should investigate the context-specific motivations for cannibalism, like nutritional stress, warfare, funerary sites, or ritual power appropriation.
Similar archeological techniques have been used to explore behaviours of cannibalism among Indigenous Huron-Wendat populations in 1651 Canada, where human bones exhibit cutmarks, perimortem fractures, and thermal modifications (Spence & Jackson, 2014). These shared taphonomic signatures across continents reveal recurring practices under ecological stress, bridging prehistoric Europe to North American contexts. Engaging with such analytical techniques opens up new ways that archeologists and anthropologists can investigate the variability in human behaviour, from nutritional crises to mortuary rituals.
Peopling of the Americas
By 25,000 years ago, our species was the only member of Homo left on Earth. Gone were the Neanderthals, Denisovans, Homo naledi, and Homo floresiensis. The range of modern Homo sapiens kept expanding eastward into—using the name given to this area by Europeans much later—the Western Hemisphere. This section will address what we know about the peopling of the Americas, from the first entry to these continents to the rapid spread of Indigenous Americans across its varied environments.
While evidence points to an ancient land bridge called Beringia that allowed people to cross from what is now northeastern Siberia into modern-day Alaska, what people did to cross this land bridge is still being investigated. For most of the 20th century, the accepted theory was the Ice-Free Corridor model. It stated that northeast Asians (East Asians and Siberians) first expanded across Beringia inland through a passage between glaciers that opened into the western Great Plains of the United States, just east of the Rocky Mountains, around 13,000 years ago (Swisher Et al. 2013). While life up north in the cold environment would have been harsh, migrating birds and an emerging forest might have provided sustenance as generations expanded through this land (Potter Et al. 2018).
However, in recent decades, researchers have accumulated evidence against the Ice-Free Corridor model. Archaeologist K. R. Fladmark (1979) brought the alternate Coastal Route model into the archaeological spotlight; researcher Jon M. Erlandson has been at the forefront of compiling support for this theory (Erlandson Et al. 2015). The new focus is the southern edge of the land bridge instead of its center: About 16,000 years ago, members of our species expanded along the coastline from northeast Asia, east through Beringia, and south down the Pacific Coast of North America while the inland was still sealed off by ice. The coast would have been free of ice at least part of the year, and many resources would have been found there, such as fish (e.g., salmon), mammals (e.g., whales, seals, and otters), and plants (e.g., seaweed).
South through the Americas
When the first modern Homo sapiens reached the Western Hemisphere, the spread through the Americas was rapid. Multiple migration waves crossed from North to South America (Posth Et al. 2018). Our species took advantage of the lack of hominin competition and the bountiful resources both along the coasts and inland. The Americas had their own wide array of megafauna, which included woolly mammoths (Figure 13.20), mastodons, camels, horses, ground sloths, giant tortoises, and—a favourite of researchers—a two-meter-tall beaver. The reason we cannot see these amazing animals today may be that resources gained from these fauna were crucial to the survival for people over 12,000 years ago (Araujo Et al. 2017). Several sites are notable for what they add to our understanding of the distant past in the Americas, including interactions with megafauna and other elements of the environment.
A 2019 discovery may allow researchers to improve theories about the peopling of the Americas. In White Sands National Park, New Mexico, 60 human footprints have been astonishingly dated to around 22,000 years ago (Bennett Et al. 2021). This date and location do not match either the Ice-Free Corridor or Coastal Route models. Researchers are now working to verify the find and adjust previous models to account for the new evidence. This groundbreaking find is sparking new theories; it is another example of the fast pace of research performed on our past.
Monte Verde is a landmark site that shows that the human population had expanded down the whole vertical stretch of the Americas to Chile by 14,600 years ago. The site has been excavated by archaeologist Tom D. Dillehay and his team (2015). The remains of nine distinct edible species of seaweed at the site shows familiarity with coastal resources and relates to the Coastal Route model by showing a connection between the inland people and the sea.
Named after the town in New Mexico, the Clovis stone-tool style is the first example of a widespread culture across much of North America, between 13,400 and 12,700 years ago (Miller, Holliday, and Bright 2013). Clovis points were fluted with two small projections, one on each end of the base, facing away from the head (Figure 13.21). The stone points found at this site match those found as far as the Canadian border and northern Mexico, and from the west coast to the east coast of the United States. Fourteen Clovis sites also contained the remains of mammoths or mastodons, suggesting that hunting megafauna with these points was an important part of life for the Clovis people. After the spread of the Clovis style, it diversified into several regional styles, keeping some of the Clovis form but also developing their own unique touches.
The Big Picture: The Assimilation Hypothesis
How do researchers make sense of all of these modern Homo sapiens discoveries that cover over 300,000 years of time and stretch across every continent except Antarctica? How was modern Homo sapiens related to archaic Homo sapiens?
The Assimilation hypothesis proposes that modern Homo sapiens evolved in Africa first and expanded out but also interbred with the archaic Homo sapiens they encountered outside Africa (Figure 13.22). This hypothesis is powerful since it explains why Africa has the oldest modern human fossils, why early modern humans found in Europe and Asia bear a resemblance to the regional archaics, and why traces of archaic DNA can be found in our genomes today (Dannemann and Racimo 2018; Reich Et al. 2010; Reich Et al. 2011; Slatkin and Racimo 2016; Smith Et al. 2017; Wall and Yoshihara Caldeira Brandt 2016).
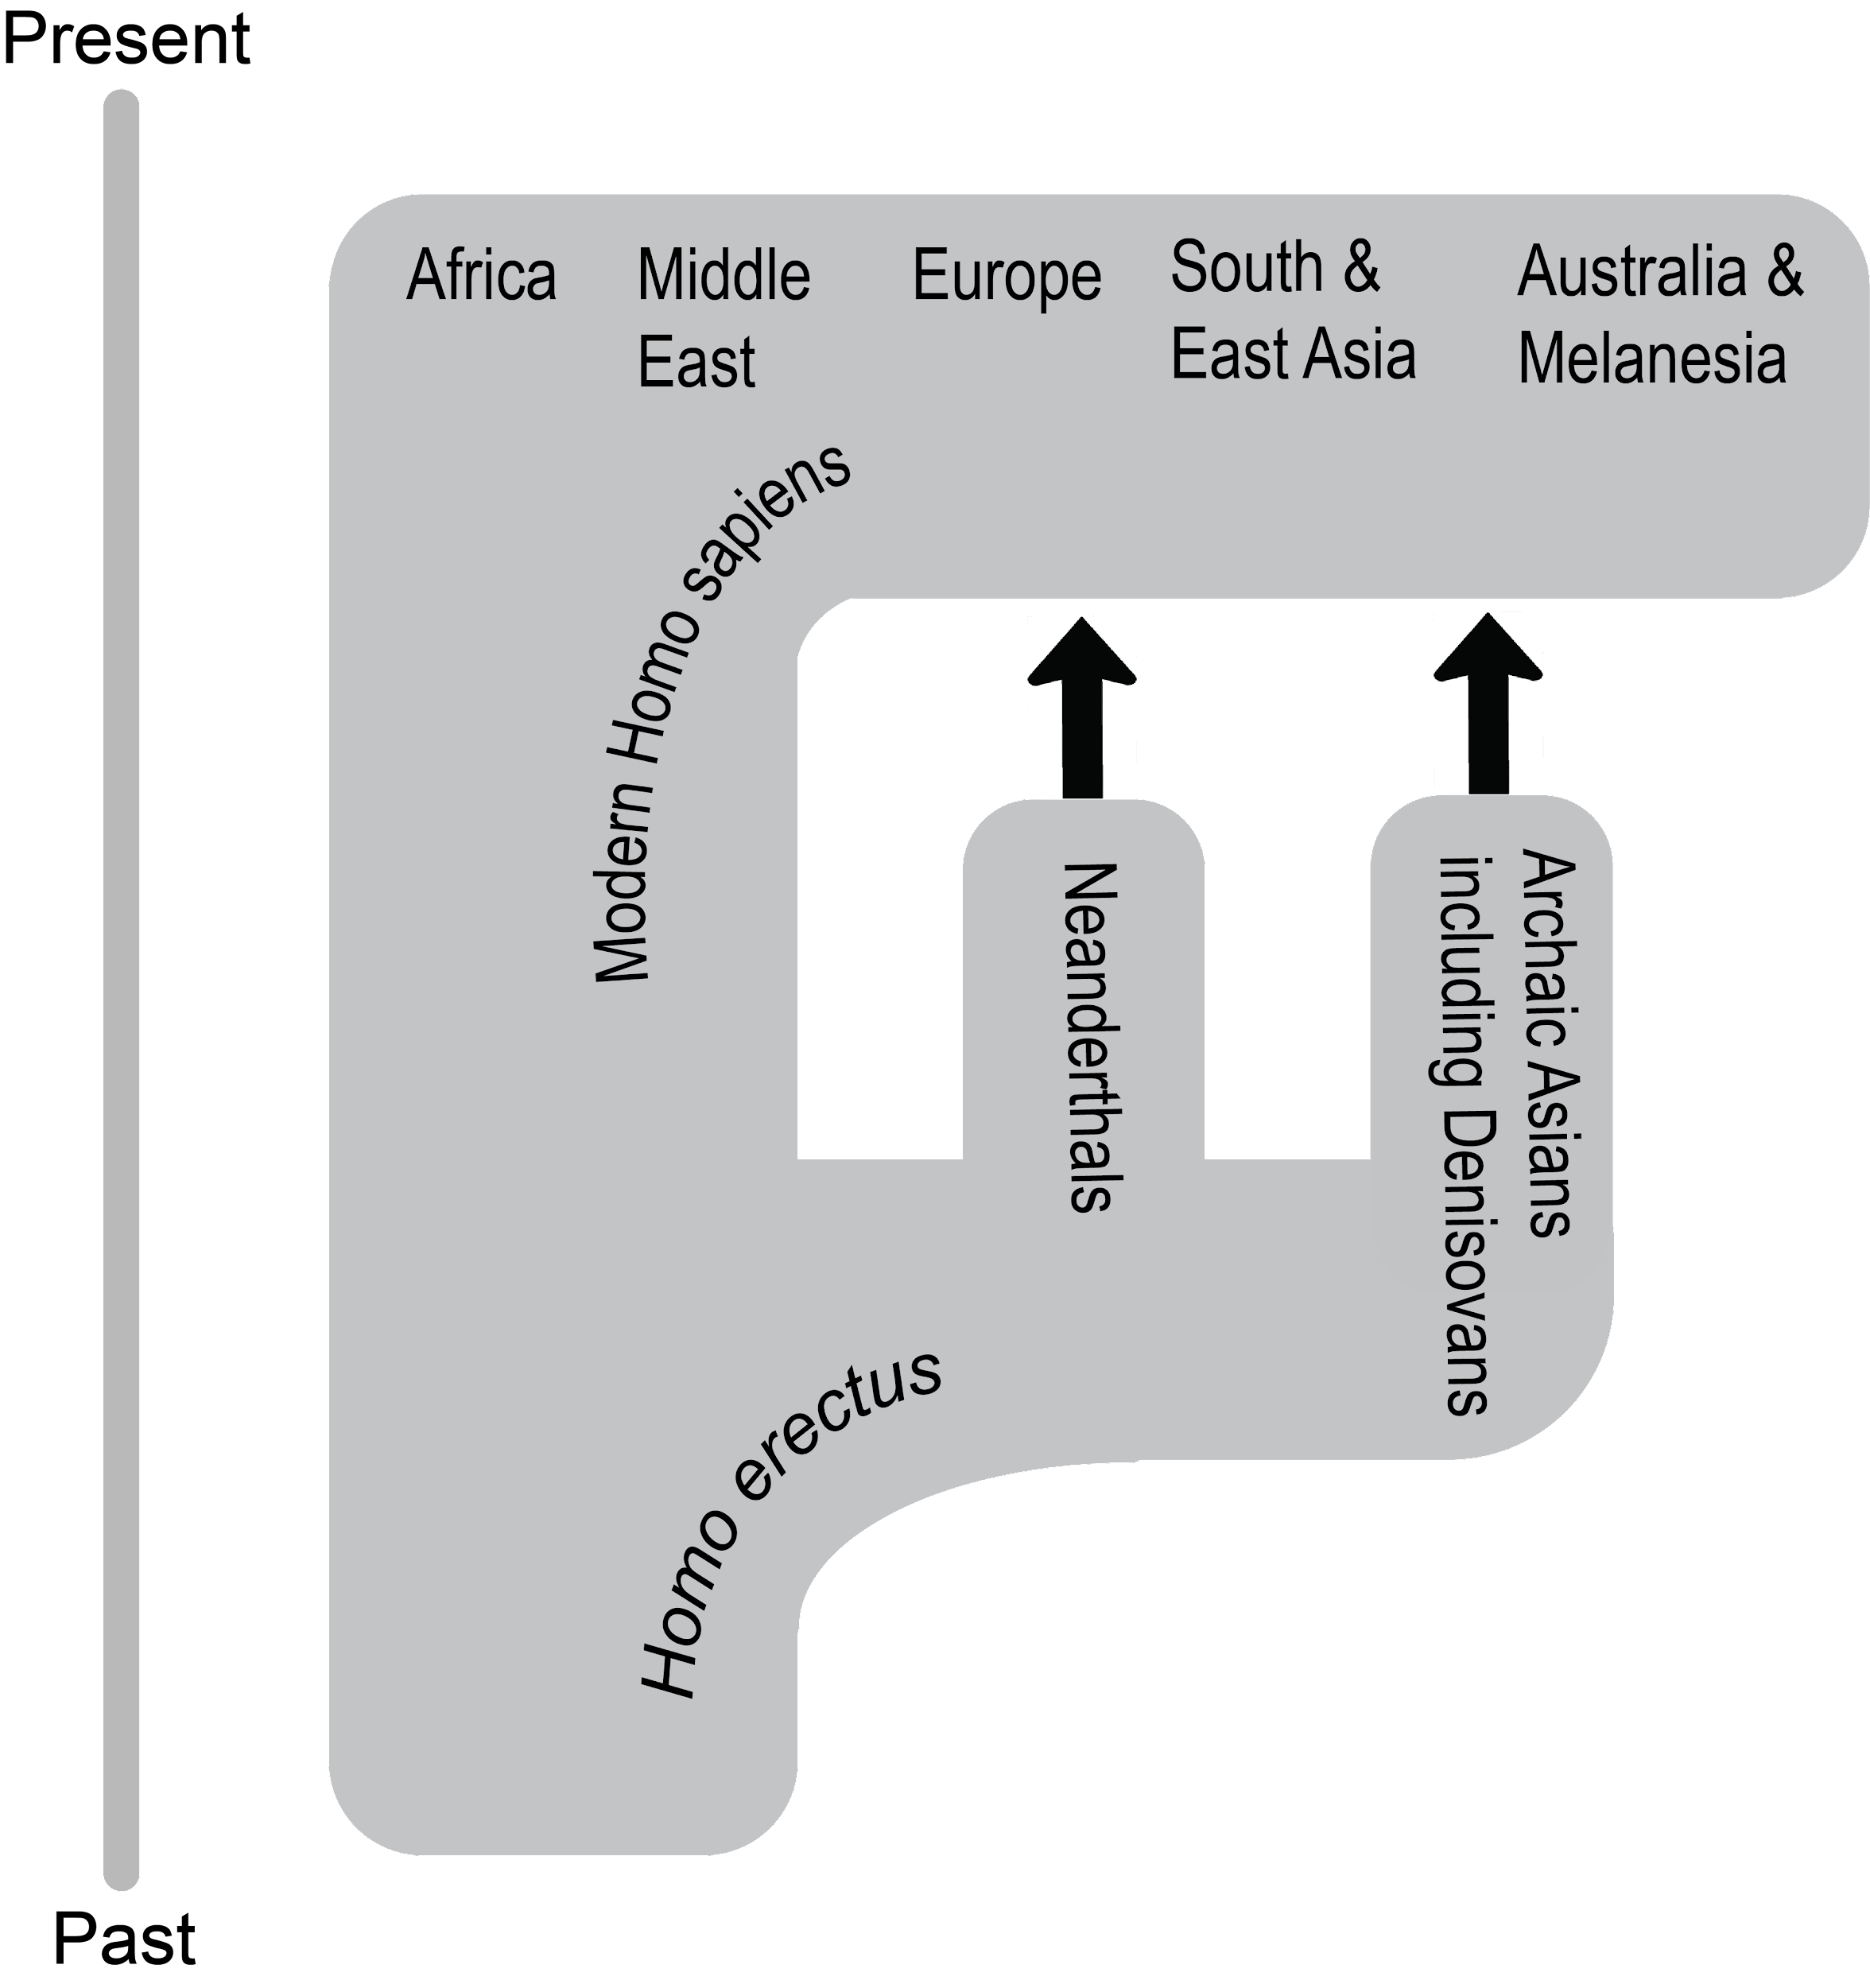
While researchers have produced a model that satisfies the data, there are still a lot of questions for paleoanthropologists to answer regarding our origins. What were the patterns of migration in each part of the world? Why did the archaic humans go extinct? In what ways did archaic and modern humans interact? The definitive explanation of how our species started and what our ancestors did is still out there to be found. You are now in a great place to welcome the next discovery about our distant past—maybe you’ll even contribute to our understanding as well.
The Chain Reaction of Agriculture
While it may be hard to imagine today, for most of our species’ existence we were nomadic: moving through the landscape without a singular home. Instead of a refrigerator or pantry stocked with food, we procured nutrition and other resources as needed based on what was available in the environment. This section gives an overview of how the foraging lifestyle enabled the expansion of our species and how the invention of a new way of life caused a chain reaction of cultural change.
The Foraging Tradition
There are a variety of possible subsistence strategies, or methods of finding sustenance and resources. To understand our species is to understand the subsistence strategy of foraging, or the search for resources in the environment. While most (but not all) humans today live in cultures that practice agriculture (whereby we greatly shape the environment to mass produce what we need), we have spent far more time as nomadic foragers than as settled agriculturalists. As such, it has been suggested that our traits have evolved to be primarily geared toward foraging. For instance, our efficient bipedalism allows persistence-hunting across long distances as well as movement from resource to resource.
How does human foraging, also known as hunting and gathering, work? Anthropologists have used all four fields to answer this question (see Ember n.d.). Typically, people formed bands, or kin-based groups of around 50 people or less (rarely over 100). A band’s organization would be egalitarian, with a flexible hierarchy based on an individual’s age, level of experience, and relationship with others. Everyone would have a general knowledge of the skills assigned to their gender roles, rather than specializing in different occupations. A band would be able to move from place to place in the environment, using knowledge of the area to forage (Figure 13.23). In varied environments—from savannas to tropical forests, deserts, coasts, and the Arctic circle—people found sustenance needed for survival.
Humans made extensive use of the foraging subsistence strategy, but this lifestyle did have limitations. The ease of foraging depended on the richness of the environment. Due to the lack of storage, resources had to be dependably found when needed. While a bountiful environment would require just a few hours of foraging a day and could lead to a focus on one location, the level and duration of labor increased greatly in poor or unreliable environments. Labor was also needed to process the acquired resources, which contributed to the foragers’ daily schedule (Crittenden and Schnorr 2017).
The adaptations to foraging found in modern Homo sapiens may explain why our species became so successful both within Africa and in the rapid expansion around the world. Overcoming the limitations, each generation at the edge of our species’s range would have found it beneficial to expand a little further, keeping contact with other bands but moving into unexplored territory where resources were more plentiful. The cumulative effect would have been the spread of modern Homo sapiens across continents and hemispheres.
Why Agriculture?
After hundreds of thousands of years of foraging, some groups of people around 12,000 years ago started to practice agriculture. This transition, called the Neolithic Revolution, occurred at the start of the Holocene epoch. While the reasons for this global change are still being investigated, two likely co-occurring causes are a growing human population and natural global climate change.
Overcrowding could have affected the success of foraging in the environment, leading to the development of a more productive subsistence strategy (Cohen 1977). Foraging works best with low population densities since each band needs a lot of space to support itself. If too many people occupy the same environment, they deplete the area faster. The high population could exceed the carrying capacity, or number of people a location can reliably support. Reaching carrying capacity on a global level due to growing population and limited areas of expansion would have been an increasingly pressing issue after the expansion through the major continents by 14,600 years ago.
A changing global climate immediately preceded the transition to agriculture, so researchers have also explored a connection between the two events. Since the Last Glacial Maximum of 23,000 years ago, the Earth slowly warmed. Then, from 13,000 to 11,700 years ago, the temperature in most of the Northern Hemisphere dropped suddenly in a phenomenon called the Younger Dryas. Glaciers returned in Europe, Asia, and North America. In Mesopotamia, which includes the Levant, the climate changed from warm and humid to cool and dry. The change would have occurred over decades, disrupting the usual nomadic patterns and subsistence of foragers around the world. The disruption to foragers due to the temperature shift could have been a factor in spurring a transition to agriculture. Researchers Gregory K. Dow and colleagues (2009) believe that foraging bands would have clustered in the new resource-rich places where people started to direct their labor to farming the limited area. After the Younger Dryas ended, people expanded out of the clusters with their agricultural knowledge (Figure 13.24).
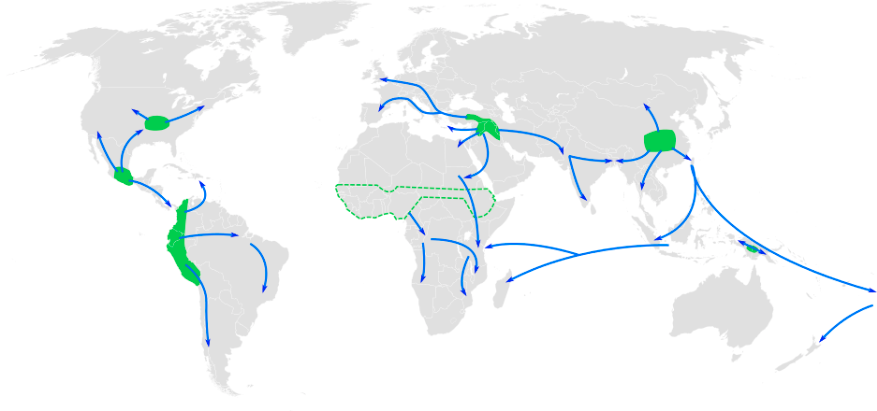
The double threat of the limitation of human continental expansion and the sudden global climate change may have placed bands in peril as more populations outpaced their environment’s carrying capacity. Not only had a growing population may have led to increased competition with other bands, but environments worldwide had shifted to create more uncertainty. As such, it has been proposed that as people in different areas around the world faced this unpredictable situation, they became the independent inventors of agriculture.
Agriculture around the World
Due to global changes to the human experience starting from 12,000 years ago, it has been suggested that cultures with no knowledge of each other turned toward intensely farming their local resources (see Figure 13.24). It is proposed that the first farmers engaged in artificial selection of their domesticates to enhance useful traits over generations. The switch to agriculture took time and effort with no guarantee of success and constant challenges (e.g. fires, droughts, diseases, and pests). The regions with the most widespread impact in the face of these obstacles became the primary centers of agriculture (Figure 13.25; Fuller 2010):
- Mesopotamia: The Fertile Crescent from the Tigris and Euphrates rivers through the Levant was where bands started to domesticate plants and animals around 12,000 years ago. The connection between the development of agriculture and the Younger Dryas was especially strong here. Farmed crops included wheat, barley, peas, and lentils. This was also where cattle, pigs, sheep, and goats were domesticated.
- South and East Asia: Multiple regions across this land had varieties of rice, millet, and soybeans by 10,000 years ago. Pigs were farmed with no connection to Mesopotamia. Chickens were also originally from this region, bred for fighting first and food second.
- New Guinea: Agriculture started here 10,000 years ago. Bananas, sugarcane, and taro were native to this island. Sweet potatoes were brought back from voyages to South America around the year C.E. 1000. No known animal farming occurred here.
- Mesoamerica: Agriculture from Central Mexico to northern South America also occurred from 10,000 years ago; it was also only plant based. Maize was a crop bred from teosinte grass, which has become one of the global staples. Beans, squash, and avocados were also grown in this region.
- The Andes: Starting around 8,000 years ago, local domesticated plants started with squash but later included potatoes, tomatoes, beans, and quinoa. Maize was brought down from Mesoamerica. The main farm animals were llamas, alpacas, and guinea pigs.
- Sub-Saharan Africa: This region went through a change 5,000 years ago called the Bantu expansion. The Bantu agriculturalists were established in West Central Africa and then expanded south and east. Native varieties of rice, yams, millet, and sorghum were grown across this area. Cattle were also domesticated here.
- Eastern North America: This region was the last major independent agriculture center, from 4,000 years ago. Squash and sunflower are the produce from this region that are most known today, though sumpweed and pitseed goosefoot were also farmed. Hunting was still the main source of animal products.
By 5,000 years ago, our species was well within the Neolithic Revolution. Agriculturalists spread to neighboring parts of the world with their domesticates, further expanding the use of this subsistence strategy. From this point, the human species changed from being primarily foragers to primarily agriculturalists with skilled control of their environments. The planet changed from mostly unaffected by human presence to being greatly transformed by humans. The revolution took millennia, but it was a true revolution as our species’ lifestyle was dramatically reshaped.
Cultural Effects of Agriculture
The worldwide adoption of agriculture altered the course of human culture and history forever. The core change in human culture due to agriculture is the move toward not moving: rather than live a nomadic lifestyle, farmers had to remain in one area to tend to their crops and livestock. The term for living bound to a certain location is sedentarism. This led to new aspects of life that were uncommon among foragers: the construction of permanent shelters and agricultural infrastructure, such as fields and irrigation, plus the development of storage technology, such as pottery, to preserve extra resources in case of future instability.
The high productivity of successful agriculture sparked further changes (Smith 2009). It is argued that since successful agriculture produced a much greater amount of food and other resources per unit of land compared to foraging, the population growth rate skyrocketed. The surplus of a bountiful harvest also provided insurance for harder times, reducing the risk of famine and bringing change to society as well. With a few farming households producing enough food to feed many others, people could start specializing in roles such as craftspeople, traders, religious figures, and artists, spurring innovation in these areas as people could now devote time and effort toward specific skills. These interdependent people would settle an area together for convenience, and over time, the growth of these settlements led to urbanization, the founding of cities that became the foci of human interaction (Figure 13.26).
The formation of cities led to new issues that sparked the growth of further specializations, called institutions. These are cultural constructs that exist beyond the individual and have wide control over a population. Leadership of these cities became hierarchical with different levels of rank and control. The stratification of society increased social inequality between those with more or less power over others. Under leadership, people built impressive monumental architecture, such as pyramids and palaces, that embodied the wealth and power of these early cities. Alliances could unite cities, forming the earliest states. In several regions of the world, state organization expanded into empires, wide-ranging political entities that covered a variety of cultures.
Urbanization brought new challenges as well. The concentration of sedentary peoples was ideal for infectious diseases to thrive since they could jump from person to person and even from livestock to person (Armelagos, Brown, and Turner 2005). While successful agriculture provided a large surplus of food to thwart famine, the food produced offered less diverse food sources than foragers’ diets (Cohen and Armelagos 1984; Cohen and Crane-Kramer 2007). This shift in nutrition caused other diseases to flourish among those who adopted farming, such as dental cavities and malocclusion (the misalignment of teeth caused by soft, agricultural diets). The need to extract “wisdom teeth” or third molars seen in agricultural cultures today stems from this misalignment between the environment our ancestors adapted to and our lifestyles today.
As the new disease trends show, the adoption of agriculture and the ensuing cultural changes were not entirely positive. It is also important to note that this is not an absolutely linear progression of human culture from simple to complex. In many cases, empires have collapsed and, in some cases, cities dispersed to low-density bands that rejected institutions. However, a global trend has emerged since the adoption of agriculture, wherein population and social inequality have increased, leading to the massive and influential nation-states of today.
The rise of states in Europe has a direct impact on many of this book’s topics. Science started as a European cultural practice by the upper class that became a standardized way to study the world. Education became an institution to provide a standardized path toward producing and gaining knowledge. The scientific study of human diversity, embroiled in the race concept that still haunts us today, was connected to the European slave trade and colonialism.
Also starting in Europe, the Industrial Revolution of the 19th century turned cities into centers of mass manufacturing and spurred the rapid development of inventions (Figure 13.27). In the technologically interconnected world of today, human society has reached a new level of complexity with globalization. In this system, goods are mass-produced and consumed in different parts of the world, weakening the reliance on local farms and factories. The imbalanced relationship between consumers and producers of goods further increases economic inequality.
As states based on agriculture and industry keep exerting influence on humanity today, there are people, like the Hadzabe of Tanzania, who continue to live a lifestyle centered on foraging. Due to the overwhelming force that agricultural societies exert, foragers today have been marginalized to live in the least habitable parts of the world—the areas that are not conducive to farming, such as tropical rainforests, deserts, and the Arctic (Headland Et al. 1989). Foragers can no longer live in the abundant environments that humans would have enjoyed before the Neolithic Revolution. Interactions with agriculturalists are typically imbalanced, with trade and other exchanges heavily favouring the larger group. One of anthropology’s important roles today is to intelligently and humanely manage equitable interactions between people of different backgrounds and levels of influence.
Special Topic: Indigenous Land Management
Insight into the lives of past modern humans has evolved as researchers revise previous theories and establish new connections with Indigenous knowledge holders.
The outdated view of foraging held that people lived off of the land without leaving an impact on the environment. Accompanying this idea was anthropologist Marshall Sahlins’s (1968) proposal that foragers were the “original affluent society” since they were meeting basic needs and achieving satisfaction with less work hours than agriculturalists and city-dwellers. This view countered an earlier idea that foragers were always on the brink of starvation. Sahlins’s theory took hold in the public eye as an attractive counterpoint to our busy contemporary lives in which we strive to meet our endless wants.
A fruitful type of study involving researchers collaborating with Indigenous experts has found that foragers did not just live off the land with minimal effort nor were they barely surviving in unchanging environments. Instead, they shaped the landscape to their needs using labor and strategies that were more subtle than what European colonizers and subsequent researchers were used to seeing. Research from two regions shows the latest developments in understanding Indigenous land management.
In British Columbia, Canada, the bridging of scientific and Indigenous perspectives has shown that the forests of the region are not untouched wilderness but, rather, have been crafted by Indigenous peoples thousands of years ago. Forest gardens adjacent to archaeological sites show higher plant diversity than unmanaged places even after 150 years (Armstrong Et al. 2021). On the coast, 3,500-year-old archaeological sites are evidence of constructed clam gardens, according to Indigenous experts (Lepofsky Et al. 2015). Another project, in consultation with Elders of the T’exelc (William Lakes First Nation) in British Columbia, introduced researchers to explanations of how forests were managed before the practice was disrupted by European colonialism (Copes-Gerbitz Et al. 2021). Careful management of controlled fires reduced the density of the forest to favour plants such as raspberries and allow easier movement through the landscape.
Similarly, the study of landscapes in Australia, in consultation with Aboriginal Australians today, shows that areas previously considered wilderness by scientists were actually the result of controlling fauna and fires. The presence of grasslands with adjacent forests were purposely constructed to attract kangaroos for hunting (Gammage 2008). People also managed other animal and insect life, from emus to caterpillars. In Tasmania, a shift from productive grassland to wildfire-prone rainforest occurred after Aboriginal Australian land management was replaced by British colonial rule (Fletcher, Hall, and Alexander 2021). The site of Budj Bim of the Gunditjmara people has archaeological features of aquaculture, or the farming of fish, that date back 6,600 years (McNiven Et al. 2012; McNiven Et al. 2015). These examples show that Indigenous knowledge of how to manipulate the environment may be invaluable at the state level, such as by creating an Aboriginal ranger program to guide modern land management.
The Future of Humanity
A common question stemming from understanding human evolution is: What will the genetic and biological traits of our species be hundreds of thousands of years in the future? When faced with this question, people tend to think of directional selection. Maybe our braincases will be even larger, resembling the large-headed and small-bodied aliens of science fiction (Figure 13.28). Or, our hands could be specialized for interacting with our touch-based technology with less risk of repetitive injury. These ideas do not stand up to scrutiny. Since natural selection is based on adaptations that increase reproductive success, any directional change must be due to a higher rate of producing successful offspring compared to other alleles. Larger brains and more agile fingers would be convenient to possess, but they do not translate into an increase in the underlying allele frequencies.
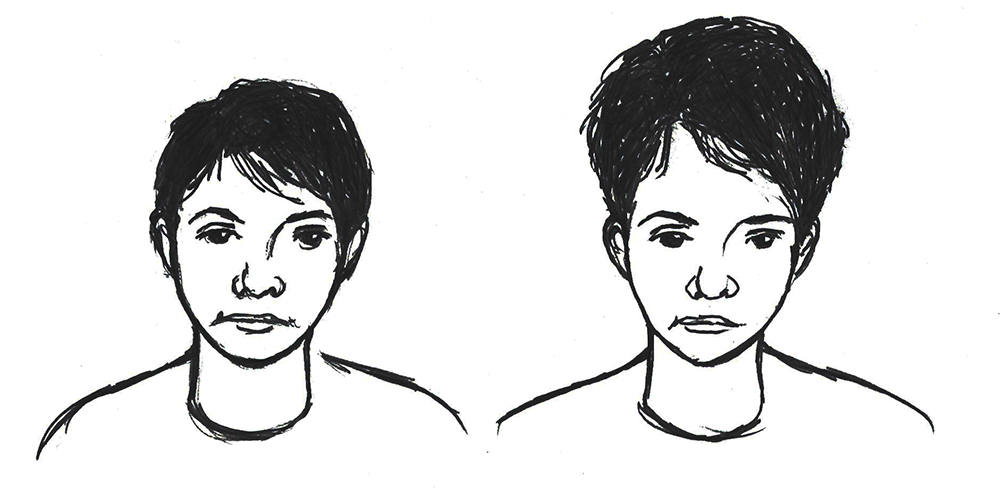
Scientists are hesitant to professionally speculate on the unknowable, and we will never know what is in store for our species one thousand or one million years from now, but there are two trends in human evolution that may carry on into the future: increased genetic variation and a reduction in regional differences.
Rather than a directional change, genetic variation in our species could expand. Our technology can protect us from extreme environments and pathogens, even if our biological traits are not tuned to handle these stressors. The rapid pace of technological advancement means that biological adaptations will become less and less relevant to reproductive success, so nonbeneficial genetic traits will be more likely to remain in the gene pool. Biological anthropologist Jay T. Stock (2008) views environmental stress as needing to defeat two layers of protection before affecting our genetics. The first layer is our cultural adaptations. Our technology and knowledge can reduce pressure on one’s genotype to be “just right” to pass to the next generation. The second defense is our flexible physiology, such as our acclimatory responses. Only stressors not handled by these powerful responses would then cause natural selection on our alleles. These shields are already substantial, and cultural adaptations will only keep increasing in strength.
The increasing ability to travel far from one’s home region means that there will be a mixing of genetic variation on a global level in the future of our species. In recent centuries, gene flow of people around the world has increased, creating admixture in populations that had been separated for tens of thousands of years. For skin colour, this means that populations all around the world could exhibit the whole range of skin colours, rather than the current pattern of decreasing melanin pigment farther from the equator. The same trend of intermixing would apply to all other traits, such as blood types. While our genetics will become more varied, the variation will be more intermixed instead of regionally isolated.
Our distant descendants will not likely be dextrous ultraintellectuals; more likely, they will be a highly variable and mobile species supported by novel cultural adaptations that make up for any inherited biological limitations. Technology may even enable the editing of DNA directly, changing these trends. With the uncertainty of our future, these are just the best-educated guesses for now. Our future is open and will be shaped little by little by the environment, our actions, and the actions of our descendants.
Hominin Species Summary
|
Hominin |
Modern Homo sapiens |
|
Dates |
315,000 years ago to present |
|
Region(s) |
Starting in Africa, then expanding around the world |
|
Famous discoveries |
Cro-Magnon individuals, discovered 1868 in Dordogne, France. Otzi the Ice Man, discovered 1991 in the Alps between Austria and Italy. Kennewick man, discovered 1996 in Washington state. |
|
Brain size |
1400 cc average |
|
Dentition |
Extremely small with short cusps. |
|
Cranial features |
An extremely globular brain case and gracile features throughout the cranium. The mandibular symphysis forms a chin at the anterior-most point. |
|
Postcranial features |
Gracile skeleton adapted for efficient bipedal locomotion at the expense of the muscular strength of most other large primates. |
|
Culture |
Extremely extensive and varied culture with many spoken and written languages. Art is ubiquitous. Technology is broad in complexity and impact on the environment. |
|
Other |
The only living hominin. Chimpanzees and bonobos are the closest living relatives. |
Summary
Modern Homo sapiens is the species that took the hominin lifestyle the furthest to become the only living member of that lineage. The largest factor that allowed us to persist while other hominins went extinct was likely our advanced ability to culturally adapt to a wide variety of environments. Our species, with its skeletal and behavioural traits, was well-suited to be generalist-specialists who successfully foraged across most of the world’s environments. The biological basis of this adaptation was our reorganized brain that facilitated innovation in cultural adaptations and intelligence for leveraging our social ties and finding ways to acquire resources from the environment. As the brain’s ability increased, it shaped the skull by reducing the evolutionary pressure to have large teeth and robust cranial bones to produce the modern Homo sapiens face.
Our ability to be generalist-specialists is seen in the geographical range that modern Homo sapiens covered in 300,000 years. In Africa, our species formed from multiregional gene flow that loosely connected archaic humans across the continent. People then expanded out to the rest of the continental Eurasia and even further to the Americas.
For most of our species’s existence, foraging was the general subsistence strategy within which people specialized to culturally adapt to their local environment. With omnivorousness and mobility, people found ways to extract and process resources, shaping the environment in return. When resource uncertainty hit the species, people around the world focused on agriculture to have a firmer control of sustenance. The new strategy shifted human history toward exponential growth and innovation, leading to our high dependence on cultural adaptations today.
While a cohesive image of our species has formed in recent years, there is still much to learn about our past. The work of many driven researchers shows that there are amazing new discoveries made all the time that refine our knowledge of human evolution. Technological innovations such as DNA analysis enable scientists to approach lingering questions from new angles. The answers we get allow us to ask even more insightful questions that will lead us to the next revelation. Like the pink limestone strata at Jebel Irhoud, previous effort has taken us so far and you are now ready to see what the next layer of discovery holds.
Review Questions
- What are the skeletal and behavioural traits that define modern Homo sapiens? What are the evolutionary explanations for its presence?
- What are some creative ways that researchers have learned about the past by studying fossils and artifacts?
- How do the discoveries mentioned in “First Africa, Then the World” fit the Assimilation model?
- What is foraging? What adaptations do we have for this subsistence strategy? Could you train to be a skilled forager?
- What are aspects of your life that come from dependence on agriculture and its cultural effects? Where did the ingredients of your favourite foods originate from?
Key Terms
African multiregionalism: The idea that modern Homo sapiens evolved as a complex web of small regional populations with sporadic gene flow among them.
Agriculture: The mass production of resources through farming and domestication.
Aquaculture: The farming of fish using techniques such as trapping, channels, and artificial ponds.
Assimilation hypothesis: Current theory of modern human origins stating that the species evolved first in Africa and interbred with archaic humans of Europe and Asia.
Atlatl: A handheld spear thrower that increased the force of thrown projectiles.
Band: A small group of people living together as foragers.
Beringia: Ancient landmass that connected Siberia and Alaska. The ancestors of Indigenous Americans would have crossed this area to reach the Americas.
Carrying capacity: The amount of organisms that an environment can reliably support.
Coastal Route model: Theory that the first Paleoindians crossed to the Americas by following the southern coast of Beringia.
Early Modern Homo sapiens, Early Anatomically Modern Human: Terms used to refer to transitional fossils between archaic and modern Homo sapiens that have a mosaic of traits. Humans like ourselves, who mostly lack archaic traits, are referred to as Late Modern Homo sapiens and simply Anatomically Modern Humans.
Egalitarian: Human organization without strict ranks. Foraging societies tend to be more egalitarian than those based on other subsistence strategies.
Foraging: Lifestyle consisting of frequent movement through the landscape and acquiring resources with minimal storage capacity.
Generalist-specialist niche: The ability to survive in a variety of environments by developing local expertise. Evolution toward this niche may have been what allowed modern Homo sapiens to expand past the geographical range of other human species.
Globalization: A recent increase in the interconnectedness and interdependence of people that is facilitated with long-distance networks.
Globular: Having a rounded appearance. Increased globularity of the braincase is a trait of modern Homo sapiens.
Gracile: Having a smooth and slender quality; the opposite of robust.
Holocene: The epoch of the Cenozoic Era starting around 12,000 years ago and lasting arguably through the present.
Ice-Free Corridor model: Theory that the first Native Americans crossed to the Americas through a passage between glaciers.
Institutions: Long-lasting and influential cultural constructs. Examples include government, organized religion, academia, and the economy.
Last Glacial Maximum: The time 23,000 years ago when the most recent ice age was the most intense.
Later Stone Age: Time period following the Middle Stone Age with a diversification in tool types, starting around 50,000 years ago.
Levant: The eastern coast of the Mediterranean. The site of early modern human expansion from Africa and later one of the centers of agriculture.
Megafauna: Large ancient animals that may have been hunted to extinction by people around the world.
Mental eminence: The chin on the mandible of modern H. sapiens. One of the defining traits of our species.
Microlith: Small stone tool found in the Later Stone Age; also called a bladelet.
Middle Stone Age: Time period known for Mousterian lithics that connects African archaic to modern Homo sapiens.
Monumental architecture: Large and labor-intensive constructions that signify the power of the elite in a sedentary society. A common type is the pyramid, a raised crafted structure topped with a point or platform.
Mosaic: Composed from a mix or composite of traits.
Neolithic Revolution: Time of rapid change to human cultures due to the invention of agriculture, starting around 12,000 years ago.
Ochre: Iron-based mineral pigment that can be a variety of yellows, reds, and browns. Used by modern human cultures worldwide since at least 80,000 years ago.
Sahul: Ancient landmass connecting New Guinea and Australia.
Sedentarism: Lifestyle based on having a stable home area; the opposite of nomadism.
Southern Dispersal model: Theory that modern H. sapiens expanded from East Africa by crossing the Red Sea and following the coast east across Asia.
Subsistence strategy: The method an organism uses to find nourishment and other resources.
Sunda: Ancient Asian landmass that incorporated modern Southeast Asia.
Supraorbital torus: The bony brow ridge across the top of the eye orbits on many hominin crania.
Upper Paleolithic: Time period considered synonymous with the Later Stone Age.
Urbanization: The increase of population density as people settled together in cities.
Wallacea: Archipelago southeast of Sunda with different biodiversity than Asia.
Younger Dryas: The rapid change in global climate—notably a cooling of the Northern Hemisphere—13,000 years ago.
For Further Exploration
Websites
First-person virtual tour of Lascaux cave with annotated cave art: Ministère de la Culture and Musée d’Archéologie Nationale. “Visit the cave” Lascaux website.
Online anthropology magazine articles related to paleoanthropology and human evolution: SAPIENS. “Evolution.” SAPIENS website.
Various presentations of information about hominin evolution: Smithsonian Institution. “What does it mean to be human?” Smithsonian National Museum of Natural History website.
Magazine-style articles on archaeology and paleoanthropology: ThoughtCo. “Archaeology.” ThoughtCo. Website.
Database of comparisons across hominins and primates: University of California, San Diego. “MOCA Domains.” Center for Academic Research & Training in Anthropogeny website.
Books
Engaging book that covers human-made changes to the environment with industrialization and globalization: Kolbert, Elizabeth. 2014. The Sixth Extinction: An Unnatural History. New York: Bloomsbury.
Overview of what human life was like among the environmental shifts of the Ice Age: Woodward, Jamie. 2014. The Ice Age: A Very Short Introduction. Oxford: OUP Press.
Articles
Recent review paper about the current state of paleoanthropology research: Stringer, C. 2016. “The Origin and Evolution of Homo sapiens.” Philosophical Transactions of the Royal Society B 371 (1698).
Overview of the history of American paleoanthropology and the many debates that have occurred over the years: Trinkaus, E. 2018. “One Hundred Years of Paleoanthropology: An American Perspective.” American Journal of Physical Anthropology 165 (4): 638–651.
Amazing magazine article that synthesizes hominin evolution and why it is important to study this subject: Wheelwright, Jeff. 2015. “Days of Dysevolution.” Discover 36 (4): 33–39.
Fascinating research on Ötzi, a mummy from 5,000 years ago: Wierer, Ursula, Simona Arrighi, Stefano Bertola, Günther Kaufmann, Benno Baumgarten, Annaluisa Pedrotti, Patrizia Pernter, and Jacques Pelegrin. 2018. “The Iceman’s Lithic Toolkit: Raw Material, Technology, Typology and Use.” PLOS One 13 (6): e0198292. https://doi.org/10.1371/journal.pone.0198292.
Documentaries
PBS NOVA series covering the expansion of modern Homo sapiens and interbreeding with archaic humans: Brown, Nicholas, dir. 2015. First Peoples. Edmonton: Wall to Wall Television. Amazon Prime Video.
PBS NOVA special featuring the footprints found in White Sands National Park: Falk, Bella, dir. 2016. Ice Age Footprints. Boston: Windfall Films. https://www.pbs.org/wgbh/nova/video/ice-age-footprints/.
PBS NOVA special about how modern humans evolved adaptations to different environments. Shows how present-day people live around the world: Thompson, Niobe, dir. 2016. Great Human Odyssey. Edmonton: Clearwater Documentary. https://www.pbs.org/wgbh/nova/evolution/great-human-odyssey.html.
References
Araujo, Bernardo B. A., Luiz Gustavo R. Oliveira-Santos, Matheus S. Lima-Ribeiro, José Alexandre F. Diniz-Filho, and Fernando A. S. Fernandez. 2017. “Bigger Kill Than Chill: The Uneven Roles of Humans and Climate on Late Quaternary Megafaunal Extinctions.” Quaternary International 431: 216–222.
Armelagos, George J., Peter J. Brown, and Bethany Turner. 2005. “Evolutionary, Historical, and Political Economic Perspectives on Health and Disease.” Social Science & Medicine 61 (4): 755–765.
Armstrong, C. G., J. E. D. Miller, A. C. McAlvay, P. M. Ritchie, and D. Lepofsky. 2021. “Historical Indigenous Land-Use Explains Plant Functional Trait Diversity. Ecology and Society 26 (2): 6.
Bar-Yosef Mayer, Daniella E., Bernard Vandermeersch, and Ofer Bar-Yosef. 2009. “Shells and Ochre in Middle Paleolithic Qafzeh Cave, Israel: Indications for Modern Behavior.” Journal of Human Evolution 56 (3): 307–314.
Barbetti, M., and H. Allen. 1972. “Prehistoric Man at Lake Mungo, Australia, by 32,000 Years Bp.” Nature 240 (5375): 46–48.
Bennett, M. R., D. Bustos, J. S. Pigati, K. B. Springer, T. M. Urban, V. T. Holliday, Sally C. Reynolds, et al. (2021). “Evidence of Humans in North America during the Last Glacial Maximum.” Science 373 (6562): 1528–1531.
Bowler, J. M., Rhys Jones, Harry Allen, and A. G. Thorne. 1970. “Pleistocene Human Remains from Australia: A Living Site and Human Cremation from Lake Mungo, Western New South Wales.” World Archaeology 2 (1): 39–60.
Brown, Peter. 1999. “The First Modern East Asians? Another Look at Upper Cave 101, Liujiang and Minatogawa 1.” In Interdisciplinary Perspectives on the Origins of the Japanese, edited by K. Omoto, 105–131. Kyoto: International Research Center for Japanese Studies.
Brown, Peter. 2000. “Australian Pleistocene Variation and the Sex of Lake Mungo 3.” Journal of Human Evolution 38 (5): 743–749.
Clarkson, Chris, Zenobia Jacobs, Ben Marwick, Richard Fullagar, Lynley Wallis, Mike Smith, Richard G. Roberts, et al. 2017. “Human Occupation of Northern Australia by 65,000 Years Ago.” Nature 547 (7663): 306–310.
Cohen, Mark Nathan. 1977. The Food Crisis in Prehistory: Overpopulation and the Origins of Agriculture. New Haven, CT: Yale University Press.
Cohen, Mark Nathan, and George J. Armelagos, eds. 1984. Paleopathology at the Origins of Agriculture. Orlando, FL: Academic Press.
Cohen, Mark Nathan, and Gillian M. M. Crane-Kramer, eds. 2007. Ancient Health: Skeletal Indicators of Agricultural and Economic Intensification. Gainesville, FL: University Press of Florida.
Copes-Gerbitz, K., S. Hagerman, and L. Daniels. 2021. “Situating Indigenous Knowledge for Resilience in Fire-Dependent Social-Ecological Systems.” Ecology and Society 26(4): 25. https://www.ecologyandsociety.org/vol26/iss4/art25/.
Coqueugniot, Hélène, Olivier Dutour, Baruch Arensburg, Henri Duday, Bernard Vandermeersch, and Anne-Marie Tillier. 2014. “Earliest Cranio-Encephalic Trauma from the Levantine Middle Palaeolithic: 3-D Reappraisal of the Qafzeh 11 Skull, Consequences of Pediatric Brain Damage on Individual Life Condition and Social Care.” PLOS ONE 9 (7): e102822.
Crittenden, Alyssa N., and Stephanie L. Schnorr. 2017. “Current Views on Hunter‐Gatherer Nutrition and the Evolution of the Human Diet.” American Journal of Physical Anthropology 162 (S63): 84–109.
d’Errico, Francesco, Lucinda Backwell, Paola Villa, Ilaria Degano, Jeannette J. Lucejko, Marion K. Bamford, Thomas F. G. Higham, Maria Perla Colombini, and Peter B. Beaumont. 2012. “Early Evidence of San Material Culture Represented by Organic Artifacts from Border Cave, South Africa.” Proceedings of the National Academy of Sciences 109 (33): 13214–13219.
d’Errico, Francesco, Christopher Henshilwood, Marian Vanhaeren, and Karen Van Niekerk. 2005. “Nassarius Kraussianus Shell Beads from Blombos Cave: Evidence for Symbolic Behaviour in the Middle Stone Age.” Journal of Human Evolution 48 (1): 3–24.
Dannemann, Michael, and Fernando Racimo. 2018. “Something Old, Something Borrowed: Admixture and Adaptation in Human Evolution.” Current Opinion in Genetics & Development 53: 1–8.
Day, M. H. 1969. “Omo Human Skeletal Remains.” Nature 222: 1135–1138.
Dillehay, Tom D., Carlos Ocampo, José Saavedra, Andre Oliveira Sawakuchi, Rodrigo M. Vega, Mario Pino, Michael B. Collins, et al. 2015. “New Archaeological Evidence for an Early Human Presence at Monte Verde, Chile.” PLOS ONE 10 (11): e0141923. doi:10.1371/journal.pone.0141923.
Dow, Gregory K., Clyde G. Reed, and Nancy Olewiler. 2009. “Climate Reversals and the Transition to Agriculture.” Journal of Economic Growth 14 (1): 27–53.
Durband, Arthur C. 2014. “Brief Communication: Artificial Cranial Modification in Kow Swamp and Cohuna.” American Journal of Physical Anthropology 155 (1): 173–178.
Ember, Carol R. N.d. “Hunter-Gatherers.” Explaining Human Culture. Human Relations Area Files. Accessed March 4, 2023. https://hraf.yale.edu/ehc/summaries/hunter-gatherers.
Erlandson, Jon M., Todd J. Braje, Kristina M. Gill, and Michael H. Graham. 2015. “Ecology of the Kelp Highway: Did Marine Resources Facilitate Human Dispersal from Northeast Asia to the Americas?” The Journal of Island and Coastal Archaeology 10 (3): 392–411.
Fladmark, K. R. 1979. “Routes: Alternate Migration Corridors for Early Man in North America.” American Antiquity 44 (1): 55–69.
Fletcher, M. S., T. Hall, and A. N. Alexandra. 2021. “The Loss of an Indigenous Constructed Landscape Following British Invasion of Australia: An Insight into the Deep Human Imprint on the Australian Landscape.” Ambio 50(1): 138–149.
Fu, Qiaomei, Mateja Hajdinjak, Oana Teodora Moldovan, Silviu Constantin, Swapan Mallick, Pontus Skoglund, Nick Patterson, et al. 2015. “An Early Modern Human from Romania with a Recent Neanderthal Ancestor.” Nature 524 (7564): 216–219.
Fuller, Dorian Q. 2010. “An Emerging Paradigm Shift in the Origins of Agriculture.” General Anthropology 17 (2): 1, 8–11.
Gammage, B. 2008. “Plain Facts: Tasmania under Aboriginal Management.” Landscape Research 33 (2): 241–254.
Germonpré, Mietje, Martina Lázničková-Galetová, and Mikhail V. Sablin. 2012. “Palaeolithic Dog Skulls at the Gravettian Předmostí Site, the Czech Republic.” Journal of Archaeological Science 39 (1): 184–202.
Gröning, Flora, Jia Liu, Michael J. Fagan, and Paul O’Higgins. 2011. “Why Do Humans Have Chins? Testing the Mechanical Significance of Modern Human Symphyseal Morphology with Finite Element Analysis.” American Journal of Physical Anthropology 144 (4): 593–606.
Harvati, Katerina. 2009. “Into Eurasia: A Geometric Morphometric Reassessment of the Upper Cave (Zhoukoudian) Specimens.” Journal of Human Evolution 57 (6): 751–762.
Headland, Thomas N., Lawrence A. Reid, M. G. Bicchieri, Charles A. Bishop, Robert Blust, Nicholas E. Flanders, Peter M. Gardner, Karl L. Hutterer, Arkadiusz Marciniak, and Robert F. Schroeder. 1989. “Hunter-Gatherers and Their Neighbors from Prehistory to the Present.” Current Anthropology 30 (1): 43–66.
Henshilwood, Christopher S., Francesco d’Errico, Karen L. van Niekerk, Yvan Coquinot, Zenobia Jacobs, Stein-Erik Lauritzen, Michel Menu, and Renata García-Moreno. 2011. “A 100,000-Year-Old Ochre-Processing Workshop at Blombos Cave, South Africa.” Science 334 (6053): 219–222.
Hershkovitz, Israel, Gerhard W. Weber, Rolf Quam, Mathieu Duval, Rainer Grün, Leslie Kinsley, Avner Ayalon, et al. 2018. “The Earliest Modern Humans Outside Africa.” Science 359 (6374): 456–459.
Hublin, Jean-Jacques, Abdelouahed Ben-Ncer, Shara E. Bailey, Sarah E. Freidline, Simon Neubauer, Matthew M. Skinner, Inga Bergmann, et al. 2017. “New Fossils from Jebel Irhoud, Morocco, and the Pan-African Origin of Homo sapiens.” Nature 546 (7657): 289–292.
Lepofsky, D., N. F. Smith, N. Cardinal, J. Harper, M. Morris, M., Gitla (Elroy White), Randy Bouchard, et al. 2015. “Ancient Shellfish Mariculture on the Northwest Coast of North America.” American Antiquity 80 (2): 236–259.
Lieberman, Daniel E. 2015. “Human Locomotion and Heat Loss: An Evolutionary Perspective.” Comprehensive Physiology 5 (1): 99–117.
Lieberman, Daniel E., Brandeis M. McBratney, and Gail Krovitz. 2002. “The Evolution and Development of Cranial Form in Homo sapiens.” Proceedings of the National Academy of Sciences 99 (3): 1134–1139.
Lieberman, Daniel E., Osbjorn M. Pearson, and Kenneth M. Mowbray. 2000. “Basicranial Influence on Overall Cranial Shape.” Journal of Human Evolution 38 (2): 291–315.
Liu, Wu, María Martinón-Torres, Yan-jun Cai, Song Xing, Hao-wen Tong, Shu-wen Pei, Mark Jan Sier, Xiao-hong Wu, R. Lawrence Edwards, and Hai Cheng. 2015. “The Earliest Unequivocally Modern Humans in Southern China.” Nature 526 (7575): 696-699.
Lucas, Peter W. 2007. “The Evolution of the Hominin Diet from a Dental Functional Perspective.” In Evolution of the Human Diet: The Known, the Unknown, and the Unknowable, edited by Peter S. Ungar, 31–38 Oxford, UK: Oxford University Press.
Marsh, W. A. & Bello, S. (2023). Cannibalism and burial in the late Upper Palaeolithic: Combining archaeological and genetic evidence. Quaternary Science Reviews, 319, 108309. https://doi.org/10.1016/j.quascirev.2023.108309
McCarthy, Robert C., and Lynn Lucas. 2014. “A Morphometric Reassessment of Bou-Vp-16/1 from Herto, Ethiopia.” Journal of Human Evolution 74: 114–117.
McDougall, Ian, Francis H. Brown, and John G. Fleagle. 2005. “Stratigraphic Placement and Age of Modern Humans from Kibish, Ethiopia.” Nature 433 (7027): 733–736.
McNiven, I. J., J. Crouch, T. Richards, N. Dolby, and G. Jacobsen. 2012. “Dating Aboriginal Stone-Walled Fishtraps at Lake Condah, Southeast Australia.” Journal of Archaeological Science 39 (2): 268–286.
McNiven, I., J. Crouch, T. Richards, K. Sniderman, N. Dolby, and G. Mirring. 2015. “Phased Redevelopment of an Ancient Gunditjmara Fish Trap over the Past 800 Years: Muldoons Trap Complex, Lake Condah, Southwestern Victoria.” Australian Archaeology 81 (1): 44–58.
Michel, Véronique, Hélène Valladas, Guanjun Shen, Wei Wang, Jian-xin Zhao, Chuan-Chou Shen, Patricia Valensi, and Christopher J. Bae. 2016. “The Earliest Modern Homo sapiens in China?” Journal of Human Evolution 101: 101–104.
Miller, D. Shane, Vance T. Holliday, and Jordon Bright. 2013. “Clovis across the Continent.” In Paleoamerican Odyssey, edited by Kelly E. Graf, Caroline V. Ketron, and Michael R. Waters, 207–220. College Station: Texas A&M University Press.
Neubauer, Simon, Jean-Jacques Hublin, and Philipp Gunz. 2018. “The Evolution of Modern Human Brain Shape.” Science Advances 4 (1): eaao5961. https://doi.org/10.1126/sciadv.aao5961.
Pearson, Osbjorn M. 2000. “Postcranial Remains and the Origin of Modern Humans.” Evolutionary Anthropology 9: 229–247.
Pearson, Osbjorn M. 2008. “Statistical and Biological Definitions of ‘Anatomically Modern’ Humans: Suggestions for a Unified Approach to Modern Morphology.” Evolutionary Anthropology: Issues, News, and Reviews 17 (1): 38–48.
Pobiner, B., Pante, M. & Keevil, T. (2023). Early Pleistocene cut marked hominin fossil from Koobi Fora, Kenya. Sci Rep, 13, 9896. https://doi.org/10.1038/s41598-023-35702-7
Pietschnig, Jakob, Lars Penke, Jelte M. Wicherts, Michael Zeiler, and Martin Voracek. 2015. “Meta-Analysis of Associations between Human Brain Volume and Intelligence Differences: How Strong Are They and What Do They Mean?” Neuroscience & Biobehavioral Reviews 57: 411–432.
Posth, Cosimo, Nathan Nakatsuka, Iosif Lazaridis, Pontus Skoglund, Swapan Mallick, Thiseas C. Lamnidis, Nadin Rohland, et al. 2018. “Reconstructing the Deep Population History of Central and South America.” Cell 175 (5): 1185–1197.
Potter, Ben A., James F. Baichtal, Alwynne B. Beaudoin, Lars Fehren-Schmitz, C. Vance Haynes, Vance T. Holliday, Charles E. Holmes, et al. 2018. “Current Evidence Allows Multiple Models for the Peopling of the Americas.” Science Advances 4 (8): eaat5473. https://doi.org/10.1126/sciadv.aat5473.
Reich, David, Richard E. Green, Martin Kircher, Johannes Krause, Nick Patterson, Eric Y. Durand, Bence Viola, et al. 2010. “Genetic History of an Archaic Hominin Group from Denisova Cave in Siberia.” Nature 468 (7327): 1053–1060.
Reich, David, Nick Patterson, Martin Kircher, Frederick Delfin, Madhusudan R. Nandineni, Irina Pugach, Albert Min-Shan Ko, et al. 2011. “Denisova Admixture and the First Modern Human Dispersals into Southeast Asia and Oceania.” American Journal of Human Genetics 89 (4): 516–528.
Richter, Daniel, Rainer Grün, Renaud Joannes-Boyau, Teresa E. Steele, Fethi Amani, Mathieu Rué, Paul Fernandes, et al. 2017. “The Age of the Hominin Fossils from Jebel Irhoud, Morocco, and the Origins of the Middle Stone Age.” Nature 546 (7657): 293–296.
Roberts, Patrick, and Brian A. Stewart. 2018. “Defining the ‘Generalist-Specialist’ Niche for Pleistocene Homo sapiens.” Nature Human Behaviour 2: 542–550.
Rougier, Helene, Ştefan Milota, Ricardo Rodrigo, Mircea Gherase, Laurenţiu Sarcinǎ, Oana Moldovan, João Zilhão, et al. 2007. “Peştera Cu Oase 2 and the Cranial Morphology of Early Modern Europeans.” Proceedings of the National Academy of Sciences 104 (4): 1165–1170.
Sahlins, Marshall. 1968. “Notes on the Original Affluent Society.” In Man the Hunter, edited by R. B. Lee and I. DeVore, 85–89. New York: Aldine Publishing Company.
Saladié, P. & Rodríguez-Hidalgo, A. (2017). Archaeological Evidence for Cannibalism in Prehistoric Western Europe: from Homo antecessor to the Bronze Age. Journal of Archaeological Method and Theory 24, 1034–1071. https://doi.org/10.1007/s10816-016-9306-y
Sawyer, G. J., and Blaine Maley. 2005. “Neanderthal Reconstructed.” The Anatomical Record (Part B: New Anat.) 283 (1): 23–31.
Scerri, Eleanor M. L., Mark G. Thomas, Andrea Manica, Philipp Gunz, Jay T. Stock, Chris Stringer, Matt Grove, et al. 2018. “Did Our Species Evolve in Subdivided Populations Across Africa, and Why Does It Matter?” Trends in Ecology & Evolution 33 (8): 582–594.
Shea, John J. 2011. “Refuting a Myth about Human Origins.” American Scientist 99 (2): 128–135.
Shea, John J., and Ofer Bar-Yosef. 2005. “Who Were the Skhul/Qafzeh People? An Archaeological Perspective on Eurasia’s Oldest Modern Humans.” Journal of the Israel Prehistoric Society 35: 451–468.
Slatkin, Montgomery, and Fernando Racimo. 2016. “Ancient DNA and Human History.” Proceedings of the National Academy of Sciences 113 (23): 6380–6387.
Smithsonian Institution. (2023, June 26). Humans’ evolutionary relatives butchered one another 1.45 million years ago. Smithsonian Institution. https://www.si.edu/newsdesk/releases/humans-evolutionary-relatives-butchered-one-another-145-million-years-ago
Smith, Fred H., James C. M. Ahern, Ivor Janković, and Ivor Karavanić. 2017. “The Assimilation Model of Modern Human Origins in Light of Current Genetic and Genomic Knowledge.” Quaternary International 450: 126–136.
Smith, Michael. 2009. “V. Gordon Childe and the Urban Revolution: A Historical Perspective on a Revolution in Urban Studies.” Town Planning Review 80 (1): 3–29.
Spence, M., & Jackson, L. J. (2014). The Bioarchaeology of Cannibalism at the Charity Site. Journal of The Ontario Archaeological Society , 94, 65–80. https://www.academia.edu/14371786/The_Bioarchaeology_of_Cannibalism_at_the_Charity_Site
Stock, Jay T. 2008. “Are Humans Still Evolving?” EMBO Reports 9 (Suppl 1): S51–S54.
Swisher, Mark E., Dennis L. Jenkins, Lionel E. Jackson Jr., and Fred M. Phillips. 2013. “A Reassessment of the Role of the Canadian Ice-Free Corridor in Light of New Geological Evidence.” Poster Symposium 5B: Geology, Geochronology and Paleoenvironments of the First Americans at the Paleoamerican Odyssey Conference, Santa Fe, New Mexico, October 16–19.
Thorne, A. G., and P. G. Macumber. 1972. “Discoveries of Late Pleistocene Man at Kow Swamp, Australia.” Nature 238 (5363): 316–319.
Trinkaus, Erik, Ştefan Milota, Ricardo Rodrigo, Gherase Mircea, and Oana Moldovan. 2003a. “Early Modern Human Cranial Remains from the Peştera Cu Oase, Romania.” Journal of Human Evolution 45 (3): 245–253.
Trinkaus, Erik, Oana Moldovan, Adrian Bîlgăr, Laurenţiu Sarcina, Sheela Athreya, Shara E Bailey, Ricardo Rodrigo, Gherase Mircea, Thomas Higham, and Christopher Bronk Ramsey. 2003b. “An Early Modern Human from the Peştera Cu Oase, Romania.” Proceedings of the National Academy of Sciences 100 (20): 11231–11236.
Ullrich, H. (2005). Cannibalistic rites within mortuary practices from the palaeolithic to middle aged in Europe. Anthropologie (1962-), 43(2/3), 249–261. http://www.jstor.org/stable/26292739
Velemínská, J., J. Brůzek, P. Velemínský, L. Bigoni, A. Sefcáková, and S. Katina. 2008. “Variability of the Upper-Palaeolithic Skulls from Predmostí Near Prerov (Czech Republic): Craniometric Comparison with Recent Human Standards.” Homo 59 (1): 1–26.
Vidal, Céline M., Christine S. Lane, Asfawossen Asrat, Dan N. Barfod, Darren F. Mark, Emma L. Tomlinson, Ambdemichael Zafu Tadesse, et al. (2022). “Age of the Oldest Known Homo sapiens from Eastern Africa. Nature 601 (7894): 579–583.
Villa, P., Bouville, C., Courtin, J., Helmer, D., Mahieu, E., Shipman, P., Belluomini, G. & Branca, M. (1986). Cannibalism in the Neolithic. Science, 233(4762), 431–437. doi:10.1126/science.233.4762.431
Villa, Paola, Sylvain Soriano, Tsenka Tsanova, Ilaria Degano, Thomas F. G. Higham, Francesco d’Errico, Lucinda Backwell, Jeannette J. Lucejko, Maria Perla Colombini, and Peter B. Beaumont. 2012. “Border Cave and the Beginning of the Later Stone Age in South Africa.” Proceedings of the National Academy of Sciences 109 (33): 13208–13213.
Wall, Jeffrey D., and Deborah Yoshihara Caldeira Brandt. 2016. “Archaic Admixture in Human History.” Current Opinion in Genetics & Development 41: 93–97.
White, Tim D., Berhane Asfaw, David DeGusta, Henry Gilbert, Gary D. Richards, Gen Suwa, and F. Clark Howell. 2003. “Pleistocene Homo sapiens from Middle Awash, Ethiopia.” Nature 423 (6941): 742–747.
Woo, Ju-Kang. 1959. “Human Fossils Found in Liukiang, Kwangsi, China.” Vertebrata PalAsiatica 3 (3): 109–118.
Wu, XiuJie, Wu Liu, Wei Dong, JieMin Que, and YanFang Wang. 2008. “The Brain Morphology of Homo Liujiang Cranium Fossil by Three-Dimensional Computed Tomography.” Chinese Science Bulletin 53 (16): 2513–2519.
Acknowledgements
I could not have undertaken this project without the help of many who got me to where I am today. I extend sincere thank yous to the many colleagues and former students who have inspired me to keep learning and talking about anthropology. Thank you also to all who are involved in this textbook project. The anonymous reviewers truly sparked improvements to the chapter. Lastly, the staff of Starbucks #5772 also contributed immensely to this text.
Natural; as in behavior that comes naturally.
The prevention or inhibition of reproduction of healthy adults.
Any time or energy a parent devotes to the current offspring that enhances its survival (and eventual reproductive success) at the expense of the parent’s ability to invest in the next offspring.
Selection for traits that enhance the ability of members of one sex to compete amongst themselves.
The idea that new behaviors can be acquired by observing and imitating others.
Raising one’s hair or fur in an effort to look bigger.
The ability to differentiate conspecifics from members of other species.
The systematic use of signals to refer to objects in the environment.
Conveying information through scent.
Having the ability to see reds, yellows, blues, greens, and ultraviolet.
A distinctive pattern of behavior shared by multiple individuals in a social group, which persists over time and is acquired through social learning.
The act of searching for food.
When an organism, which is limited in the time and energy it can put into aspects of its biology and behavior, is shaped by natural selection to invest in one adaptation at the expense of another.
A grouping based on overall similarity in lifestyle, appearance, and behavior.
A trait that has been recently modified, most helpful when assigning taxonomic classification.
A trait that has been modified for a specific purpose.
Having thumbs and toes that go in a different direction from the rest of the fingers, allows for grasping with hands and feet.
A bony plate that provides protection to the side and back of the eye.
A descriptor for an organism that spends most of its time in trees.